Showing posts with label Neanderthals. Show all posts

Monday, April 2, 2018

Africa's Neanderthals


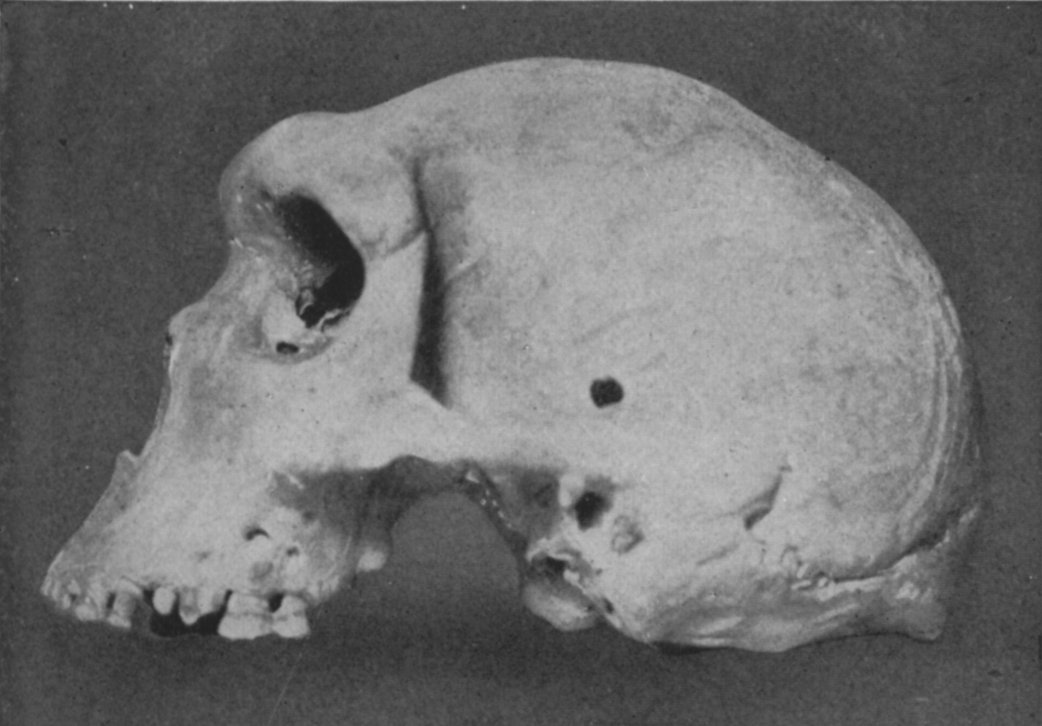
Skull from Zambia, dated to 110,000 years ago. Modern humans co-existed with archaic groups in Africa, particularly in the south and west.


When and where did modern humans emerge? Anatomical evidence points to somewhere in eastern Africa some 300,000 years ago. The time of origin is different if we look at behavioral and genetic evidence. Sophisticated tool-making, detailed artwork, and other signs of “behavioral modernity” appeared only 70,000 years ago (Brown et al., 2012). Genetic evidence points to a series of demographic expansions between 80,000 and 60,000 years ago in eastern Africa, with the last one spreading throughout Africa and into Eurasia (Watson et al. 1997). At that moment, an innovation in thinking seems to have given these truly modern humans an edge over everyone else.

As these humans spread throughout the world, to what extent did they intermix with the more archaic groups they replaced? We can answer this question for Eurasia by comparing the modern human genome with reconstructed genomes of the now-extinct Neanderthals (Europe, Middle East, and Central Asia) and Denisovans (East Asia, Southeast Asia). Present-day Eurasians have relatively low levels of archaic admixture: about 2% from Neanderthals and up to 5% from Denisovans (Sankararaman et al. 2016).

What about Africa? Unfortunately, we have not yet reconstructed the genome of any archaic population from that continent. We probably never will, given that DNA tends to degrade quickly in tropical climates. In theory, there should be more admixture in Africa than in Eurasia, since many archaic Africans would have been "near-modern," i.e., much more similar in appearance, behavior, and genetic makeup to modern humans than either Neanderthals or Denisovans. Greater genetic similarity would have also made hybrid infertility less likely. Indeed, it looks like male fertility suffered from hybridization with Neanderthals or Denisovans, given that present-day humans have a lower proportion of archaic ancestry on the X chromosome and in genes disproportionately expressed in the testes (Sankararaman et al. 2016). In these parts of the genome, natural selection has stepped in to remove archaic admixture.

The above speculations seem borne out by a recent and still unpublished paper. Its authors, Sriram Sankararaman and Arun Durvasula, came up with a novel way to measure admixture from an unknown archaic group, essentially by using a machine learning algorithm (which they validated with data on Neanderthal introgression in present-day Europeans). When they applied this method to Yoruba from Nigeria, they found a level of archaic admixture higher than in any other human population known to date:

Our results suggest that Yoruban individuals trace about 7.9% of their genomes to an as yet unidentified archaic population. This is in agreement with some results from previous papers in other African populations such as the Biaka and the Baka, suggesting that there was a rich diversity of hominin species within Africa and that introgression was commonplace. (Sankararaman and Durvasula 2018)

This finding is consistent with previous archaeological and genetic evidence, particularly from western and southern Africa. Both regions seem to have had archaic populations until recent times:

- A skull from a Nigerian site (Iwo Eleru) is only about 16,300 years old and yet looks intermediate in shape between modern humans on the one hand and Neanderthals and Homo erectus on the other. It resembles the skull of a near-modern human, like the Skhul-Qafzeh hominins who lived in the Middle East some 80,000 to 100,000 years ago (Harvati et al., 2011; Stojanowski, 2014).

- Genomic analysis of 16 prehistoric Africans suggests that modern humans spread out of eastern Africa and into western Africa, where they mixed with an archaic population as divergent from modern humans as Neanderthals were, the time of separation from modern humans being 200,000 to 300,000 years ago. This archaic admixture is estimated at 9% in Yoruba and 13% in Mende (Skoglund et al. 2017)

- Genomic analysis shows an apparently higher level of Neanderthal ancestry in the Yoruba of Nigeria than in the Luhya of Kenya. This admixture seems to come from a Neanderthal-like population that formerly lived in West Africa (Hawks 2012)

- A skull from Zambia has been dated to 110,000 years ago and yet looks very much like a Homo erectus (Bada et al., 1974; Stringer, 2011). 

-  About 2% of the current African gene pool comes from a population that split from ancestral modern humans some 700,000 years ago. This archaic DNA was then picked up by modern African humans about 35,000 years ago, probably in central Africa because this admixture is highest in pygmy groups from that region (Hammer et al. 2011).

- Genomic analysis of western African pygmies (Biaka and Baka) indicates frequent, low-level interbreeding between archaic and modern humans, including an admixture event within the last 30,000 years (Hsieh et al. 2016). 

- Jawbone fragments from South Africa exhibits significant size and morphological variability, indicating admixture with an archaic population. The fragments fall within the range of 110,000 to 60,000 years ago (Malekfar, 2012)

- Sub-Saharan Africans exhibit dental traits that distinguish them from other modern humans (Sub-Saharan African Dental Complex). These traits are shared with extinct hominids and many extinct and extant nonhuman primates (Irish 1998). When dentitions are compared from western, central, eastern, and southern Africans, these ancestral traits appear to be least present in Kenyans and Tanzanians (Irish 1998). The SSADC thus seems least present in the "homeland" of modern humans (eastern Africa) and more present farther west and south.

Is the estimate of 7.9% archaic admixture a lower bound?

While the new finding of 7.9% archaic admixture is higher than what we see in other modern humans, the actual figure may be higher still. Sankararaman and Durvasula attribute this 7.9% admixture to "a deeply-diverged archaic population," while nonetheless acknowledging the "rich diversity of hominin species within Africa." Dienekes (2018) likewise notes that multiple admixture events had occurred between modern African humans and a range of "Palaeoafrican" groups.

Thus, Sankararaman and Durvasula are measuring admixture only from a highly divergent archaic group, apparently the same one that Skoglund et al. (2017) found in their study of the Yoruba. Indeed, the two studies found almost the same level of archaic admixture in the Yoruba: 7.9% versus 9%. Although Sankararaman and Durvasula validated their methodology with data on Neanderthal admixture in Europe, the two situations are not really comparable. In Europe, modern humans encountered only one archaic group over a relatively short time span, intermixture taking place essentially between 60,000 and 50,000 years ago with a second event more than 37,000 years ago (Yang and Fu 2018).  In Africa, modern humans likely encountered a range of archaic groups over a longer time, including "near-moderns" whose ancestors diverged from those of modern humans less than 200,000 years ago.

If we include introgression from these “near-moderns,” the total for archaic admixture in present-day sub-Saharan Africans should be much higher.  Indeed, 13% of the sub-Saharan gene pool seems to come from a demographic expansion that took place some 111,000 years ago and which probably brought the Skhul-Qafzeh hominins to the Middle East (Watson et al. 1997). Those hominins were anatomically modern, or almost so, but culturally Neanderthal.

Did archaic admixture help or hinder?

Mainstream evolutionary theorists have argued that admixture does more harm than good. As Ernst Mayr (1970, p. 80) wrote:

The claim has been made that species owe much of their genetic variability to introgressive hybridization. However, all the evidence contradicts this conclusion so far as animals is concerned. Not only are F1 hybrids between good species very rare, but where they occur the hybrids (even when not sterile) are demonstrably of inferior viability. The few genes that occasionally introgress into the parental species are not coadapted [...] and are selected against. Introgressive hybridization seems to be a negligible source of genetic variation in animals.

This view has been challenged by Hawks et al. (2007), who argue that gene introgression helped modern humans adapt to new environments. Instead of starting from scratch, they could cherry-pick genes that had already been tried and proven by the populations they were replacing: 

Compared with novel mutations, archaic genetic variants would have had several qualities that, in some cases, may have enhanced their selective value. Because they had long existed within human populations, these alleles had a much lower chance of being strongly deleterious. [...] Alleles with local advantages might never have been selected within the expanding modern population until it reached new climatic regimens. The spread of modern humans may have attained a burst of evolutionary change by drawing on the fruits of the existing adaptations of archaic humans. (Hawks et al. 2007)

The latest findings seem to lie between the above two views. Introgression can in some cases provide useful genes. Usually, however, it’s maladaptive.

We observe a decrease in the frequency of archaic ancestry in the Yoruban populations in more constrained regions of the genome, suggesting that these archaic alleles have been subject to the effects of purifying selection similar to the deleterious consequences of Neanderthal and Denisovan alleles in the modern human genetic background. On the other hand, we find several loci that harbor archaic haplotypes at elevated frequencies (>60%). (Sankararaman and Durvasula 2018)

Similarly, Yang and Fu (2018) note that a "gradual decline in archaic ancestry in Europeans dating from ~37 to 14 ka suggests that purifying selection lowered the amount of Neanderthal ancestry first introduced into ancient modern humans."

This pattern is consistent with findings from nonhuman species. A study of admixture in trout found sharp declines in fitness even with 20% admixture. The decline has two causes:

Hybridization can reduce fitness by either introducing alleles to a population that are not suited to the local environment (extrinsic outbreeding depression) or disrupting co-adapted gene complexes (intrinsic outbreeding depression) (Templeton 1986). These mechanisms are not mutually exclusive, and identifying the contribution of each effect is difficult. However, the high reproductive success of F1 hybrids relative to post-F1 hybrids with similar amounts of admixture suggests that some of the outbreeding depression is intrinsic. (Muhlfeld et al. 2009)

By disrupting co-adapted gene complexes, introgression causes individual genes to lose their adaptive value. Selection will thus eliminate either the introgressed alleles or the previously existing ones. In the second scenario, the complex of co-adapted genes is replaced with a simpler version.

Conclusion

Something “clicked” in eastern Africa 80,000 to 60,000 years ago. A relatively small group of humans acquired a new way of imagining themselves, each other, and the world around them, and this innovation gave them an edge over everyone else. The result: a “big bang” of population growth. They began to spread outward, first within Africa and then into Eurasia.

Their expansion within Africa seems to have proceeded more slowly than in Eurasia. Initially, these modern humans were replacing “near-moderns”—people fairly similar in appearance and genetic makeup. As they pushed farther east and south, however, they encountered populations that were much less similar. West Africa seems to have been home to a people who were as different from modern humans as Neanderthals were, perhaps being related to them. In southern Africa, modern humans encountered people even more divergent: a relic Homo erectus population. Even these highly divergent archaic groups were not rapidly replaced; they may have persisted as late as 15,000 years ago in West Africa and 30,000 years ago in central Africa. Thus, modern and archaic groups seem to have long coexisted in parts of Africa.

In general, archaic admixture reduced fitness: “archaic alleles that introgressed into the Yoruban population were deleterious on average”; neutral alleles were more likely to be retained than those that had functional impacts (Sankararaman and Durvasula 2018). A few, however, seem to have been favored by selection. This is the case with alleles located at a tumor suppressor gene, a gene involved with hormone regulation, and a gene involved with potassium channels. These are individual genes, however, and it is hard to know the impact on co-adapted gene complexes. In theory, archaic admixture should have had a disruptive effect.

Present-day Africans thus have admixture from a range of archaic groups, some being similar to modern humans and others more like Neanderthals or even Homo erectus. This admixture is highest in western and southern Africa and lowest in eastern Africa. In West Africa, admixture from a Neanderthal-like group is estimated at 7.9% by Sankararaman and Durvasula (2018) and at 9 to 13% by Skoglund et al. (2017). Admixture from “near-moderns” is harder to measure. There seems to be a 13% pan-African admixture from a population that had expanded across much of the continent some 111,000 years ago and which perhaps spilled into the Middle East, giving rise to the Skhul-Qafzeh hominins, i.e., early modern humans with Neanderthal culture (Watson et al. 1997, see L1i in Table 2).


References

Bada, J.L., R.A. Schroeder, R. Protsch, & R. Berger. (1974). Concordance of Collagen-Based Radiocarbon and Aspartic-Acid Racemization Ages, Proceedings of the National Academy of Sciences (USA) 71: 914-917.
http://www.pnas.org/content/71/3/914.short

Brown, Kyle S.; Marean, Curtis W.; Jacobs, Zenobia; Schoville, Benjamin J.; Oestmo, Simen; Fisher, Erich C.; Bernatchez, Jocelyn; Karkanas, Panagiotis; Matthews, Thalassa (2012). An early and enduring advanced technology originating 71,000 years ago in South Africa. Nature 491 (7425): 590.
https://www.researchgate.net/publication/233331522_An_early_and_enduring_advanced_technology_originating_71000_years_ago_in_South_Africa

Dienekes (2018). Statistical Palaeoafricans, Dienekes' Anthropology Blog, March 25
http://dienekes.blogspot.ca/2018/03/statistical-palaeoafricans.html

Durvasula, A., and S. Sankararaman. (2018). Recovering signals of ghost archaic admixture in the genomes of present-day Africans, BioRxiv, March 21
https://www.biorxiv.org/content/early/2018/03/21/285734  

Hammer, M.F., A.E. Woerner, F.L. Mendez, J.C. Watkins, and J.D. Wall. (2011). Genetic evidence for archaic admixture in Africa, Proceedings of the National Academy of Sciences (USA) 108: 15123-15128.
http://www.u.arizona.edu/~flmendez/papers/Hammer_2011.pdf

Harvati, K., C. Stringer, R. Grün, M. Aubert, P. Allsworth-Jones, C.A. Folorunso. (2011). The Later Stone Age Calvaria from Iwo Eleru, Nigeria: Morphology and Chronology. PLoS ONE 6(9): e24024. doi:10.1371/journal.pone.0024024
http://www.plosone.org/article/info%3Adoi%2F10.1371%2Fjournal.pone.0024024

Hawks, J. (2012). Which population in the 1000 Genomes Project samples has the most Neandertal similarity? John Hawks Weblog, February 8
http://johnhawks.net/weblog/reviews/neandertals/neandertal_dna/1000-genomes-introgression-among-populations-2012.html

Hawks, J., G. Cochran, H.C. Harpending, and B.T. Lahn. (2007). A genetic legacy from archaic Homo, Trends in Genetics 24(1): 19-23
https://s3.amazonaws.com/academia.edu.documents/46568403/A_genetic_legacy_from_archaic_Homo20160617-13508-1nt7amy.pdf?AWSAccessKeyId=AKIAIWOWYYGZ2Y53UL3A&Expires=1522259324&Signature=Ng%2FyAWbzdtcjUJ%2BDAJTY7yE8FuA%3D&response-content-disposition=inline%3B%20filename%3DA_genetic_legacy_from_archaic_Homo.pdf

Hsieh, P., A.W. Woerner, J.D. Wall, J. Lachance, S.A. Tishkoff, R.N. Gutenkunst, and M.F. Hammer. (2016). Model-based analyses of whole-genome data reveal a complex evolutionary history involving archaic introgression in Central African Pygmies. Genome Research 26(3): 291-300
https://www.ncbi.nlm.nih.gov/pmc/articles/PMC4772012/

Irish, J.D. (1998). Ancestral dental traits in recent Sub-Saharan Africans and the origins of modern humans, Journal of Human Evolution 34: 81-98.
https://www.sciencedirect.com/science/article/pii/S0047248497901913

Malekfar, L. (2012). An analysis of the Klasies River hominins using a hybrid model, American Journal of Physical Anthropology, Program of the 81st Annual Meeting of the American Association of Physical Anthropologists, p. 201.
https://s3.amazonaws.com/academia.edu.documents/33649075/anthro_poster_lily_%281%29.pdf?AWSAccessKeyId=AKIAIWOWYYGZ2Y53UL3A&Expires=1522334949&Signature=h10VLn2RDPu8HtH4X55L64S2ODU%3D&response-content-disposition=inline%3B%20filename%3DPoster_An_Analysis_of_the_Klasies_River.pdf

Mayr, E. (1970). Populations, Species, and Evolution, Belknap Press: Cambridge (Mass.)

Muhlfeld, C.C.,  S.T Kalinowski, T.E. McMahon, M.L. Taper, S. Painter, R.F. Leary, F.W. Allendorf. (2009). Hybridization rapidly reduces fitness of a native trout in the wild, Biology Letters, March 18
http://rsbl.royalsocietypublishing.org/content/early/2009/03/13/rsbl.2009.0033.short

Sankararaman, S., S. Mallick, N. Patterson, and D. Reich. (2016). The combined landscape of Denisovan and Neanderthal ancestry in present-day humans, Current Biology 26(9): 1241-1247.
https://www.sciencedirect.com/science/article/pii/S0960982216302470#bib1

Skoglund, P., J.C. Thompson, M.E. Prendergast, A. Mittnik, K. Sirak, et al. (2017). Reconstructing Prehistoric African Population Structure, Cell 171(1): 59-71
http://www.cell.com/cell/fulltext/S0092-8674(17)31008-5

Stojanowski, C.M. (2014). Iwo Eleru's place among Late Pleistocene and Early Holocene populations of North and East Africa, Journal of Human Evolution 75: 80-89.
http://www.sciencedirect.com/science/article/pii/S0047248414000876

Stringer, C. (2011). The chronological and evolutionary position of the Broken Hill cranium. American Journal of Physical Anthropology 144(supp. 52): 287

Watson, E., P. Forster, M. Richards, and H-J. Bandelt. (1997). Mitochondrial footprints of human expansions in Africa, American Journal of Human Genetics 61: 691-704. 0024024
https://www.sciencedirect.com/science/article/pii/S000292970764333X

Yang, M.A., and Q. Fu. (2018). Insights into Modern Human Prehistory Using Ancient Genomes, Trends in Genetics 34(3): 184-196
https://www.sciencedirect.com/science/article/pii/S016895251730210X

Thursday, January 4, 2018

Red-haired women are special


The Damsel of the Sanct Grael – Dante Gabriel Rossetti (1828-1882)


It's known that red-haired women, but not red-haired men, are more sensitive to pain. Red hair is also associated with a higher risk of developing endometriosis, Parkinson's disease, and decreased platelet function.

A study in the latest issue of PLoS One has confirmed that red hair, especially in women, is linked to certain health issues. According to a survey of over seven thousand participants, red-haired women do worse than other women in ten health categories and better in only three, being especially prone to colorectal, cervical, uterine, and ovarian cancer. Red-haired men seem to be as healthy as other men, doing better in three categories and worse in three. Reproductive success, i.e., number of children, is the only category where redheads of both sexes do better than other participants.

This study has also confirmed that red hair is naturally more frequent in women than in men. To a lesser degree, the same is true for blond hair and green eyes. These bright colors seem to result from a selection pressure that mainly targeted women, i.e., sexual selection. In other words, among early Europeans there were too many women and not enough men; hence, competition between women for mates favored those who could better catch the attention of men, such as through a palette of bright hair and eye colors.

Because women are overrepresented among redheads, it may be that estrogen promotes synthesis of red pigments by hair follicles, particularly during fetal development. Thus, if a baby is born red-haired and female, estrogenization of its body tissues should be, on average, near the top end of the normal range. It will therefore be more at risk of developing certain health issues.

Another hypothesis can be put forward. If red hair was the last hair color to evolve, the underlying alleles may not have finished adapting to the rest of the genome, and vice versa. This reciprocal adaptation is all the more necessary because one of the five alleles for red hair seems to be of Neanderthal origin. The hypothesis of incomplete adaptation does not exclude the hypothesis of high estrogenization. In fact, there may be interaction between the two factors. Although it's likely that sexual selection did produce new hair and eye colors, we must still explain why, in this palette of colors, red hair seems to show the greatest difference between men and women both in population frequency and in associated health effects. 


Reference

Frost P, Kleisner K, Flegr J (2017) Health status by gender, hair color, and eye color: Red-haired women are the most divergent. PLoS ONE 12(12): e0190238. 


----------------------------------------------------------------------------------


La rousse est particulière


On sait que les rousses, mais pas les roux, sont plus sensibles que les autres à la douleur. La rousseur est également associée à un plus grand risque de développer l'endométriose, la maladie de Parkinson, ainsi que des troubles de l'agrégation plaquettaire.

Une étude publiée dans le dernier numéro de la revue PLoS ONE confirme que la rousseur, surtout chez la femme, est reliée à certains problèmes de santé. Selon une enquête menée auprès de plus de sept mille participants, les rousses se classent pire que les autres femmes dans dix catégories de santé et mieux dans seulement trois, étant surtout susceptibles de développer des cancers du gros intestin, du col utérin, de l'utérus ou des ovaires. Quant aux roux, leur état de santé ressemble à celui des autres hommes : mieux dans trois catégories et pire dans trois. Le succès reproducteur, soit le nombre d'enfants, est la seule catégorie où les têtes rouges des deux sexes font mieux que les autres participants.

Cette étude confirme également que la rousseur est naturellement plus fréquente chez la femme que chez l'homme. Dans une moindre mesure,  c'est le même constat avec la blondeur et les yeux verts. Ces couleurs vives semblent être le résultat d'une pression de sélection visant surtout la femme, soit la sélection sexuelle. Autrement dit, il y aurait eu trop de femmes et pas assez d'hommes chez les premiers Européens, avec pour résultat une concurrence entre les femmes favorisant celles qui attiraient mieux les regards des hommes, comme par exemple par une palette de couleurs vives décorant les cheveux et les yeux.

Les femmes étant surreprésentées parmi les têtes rouges, on peut émettre l'hypothèse que l'œstrogène favorise la synthèse de pigments rouges dans les follicules pileux, particulièrement au cours du développement fœtal. Alors, si un enfant nait à la fois roux et de sexe féminin, l'œstrogénisation de ses tissus organiques doit être, en moyenne, vers la limite supérieure de la normale. La rousse sera donc plus à risque de connaitre certains problèmes de santé.

Une autre hypothèse est possible. Si la rousseur a été la dernière couleur de cheveux à paraître, il se peut que les allèles sous-jacents n’aient pas encore fini de s'adapter au reste du génome et vice versa. Cette adaptation réciproque est d'autant plus nécessaire parce que l'un des cinq allèles pour la rousseur semble être d'origine néandertalienne. Notons que l'hypothèse d'adaptation incomplète n'exclut pas celle de forte œstrogénisation. En fait, il pourrait y avoir une interaction entre les deux facteurs. S'il est vraisemblable que la sélection sexuelle ait produit de nouvelles couleurs des cheveux et des yeux, il faudra toujours expliquer pourquoi, dans cette palette de couleurs, la rousseur semble montrer la plus grande différence entre les hommes et les femmes, autant en termes de fréquence dans la population que sur le plan de la santé. 

Tuesday, September 26, 2017

Tales from old bones


Around three thousand years ago Bantu began to spread east and south from the Nigeria/Cameroun border, eventually replacing the original inhabitants of eastern and southern Africa. Those people no longer exist. Only the DNA in their skeletal remains are left to speak for them.


When scientists began to retrieve ancient DNA from human remains, they succeeded only at sites in the temperate and arctic zones. It seemed impossible to retrieve any at tropical sites, apparently because warm year-round temperatures soon reduce DNA to a meaningless molecular jumble.

This problem seems to be solved. Two years ago, DNA was successfully retrieved from 4,500 year old remains in Ethiopia. Now, we have ancient DNA from several sites across eastern and southern Africa over a range of dates from 10,000 to 400 years ago (Skoglund et al. 2017).

Vanished peoples

This new study shows that eastern and southern Africans have changed a lot since the time of the ancient Greeks. As far north as Tanzania, the continent was once home to peoples related to the Hottentots (now called Khoisans, Khoe-Sans, or simply San)—short in stature, gracile in body build, and light yellowish brown in color. From Zanzibar north, people were of mixed Middle Eastern and Cushitic origin—sort of like present-day Ethiopians but with more Arab ancestry.

What happened to these peoples? They were either replaced or absorbed by Bantus moving in from the west, although it now looks like they were replaced a lot more than they were absorbed. No trace of them remains in Malawi's gene pool:


Population replacement by incoming food producers appears to have been nearly complete in Malawi, where we detect little if any ancestry from the ancient individuals who lived ~8,100-2,500 BP. Instead, present-day Malawian individuals are consistent with deriving all their ancestry from the Bantu expansion of ultimate western African origin. (Skoglund et al. 2017)

The original inhabitants were related to present-day Khoisans but had significantly diverged from them:

Notably, the Khoe-San-related ancestry in ancient individuals from Malawi and Tanzania is symmetrically related to the two previously identified lineages present in the San [...], estimated to have diverged at least 20,000 years ago [...], implying that this was an ancient divergent branch of this group that lived in eastern Africa at least until 1,400 BP. (Skoglund et al. 2017)

This is in line with previous DNA findings from the Fwe (a Bantu group of southwestern Zambia), particularly the presence of Khoisan admixture that resembles nothing in present-day Khoisans:

[It is possible] that the Fwe intermarried with a Khoisan group whose genetic composition differed from that of the populations included in molecular anthropological investigations to date. [...] it is plausible that the Fwe ancestors interacted with a Khoisan community that differed genetically from those still settled in southern Africa today, which was ultimately replaced by the newcomers. (Barbieri et al. 2013)

Aside from these scattered fragments of DNA, we also have the testimony of ancient observers. Two tenth-century Arab geographers state that "in the outer reaches of the land of the Zanj there are cool highlands in which live white Zanj" (Lewis 1990, p. 121, n. 3). The Zanj are the dark-skinned peoples of east Africa and the term 'white' is better translated by 'lighter-skinned.' (The words 'black' and 'white' are often used in a relative sense in Arabic). The highlands might be the Drakensberg Escarpment of South Africa. 

Encounters with the archaic Other

Modern humans arose some 80,000 years ago in eastern Africa through a series of population expansions that culminated twenty thousand years later in a big bang that spread outward in Africa and then into the Middle East, Europe, and Asia (Watson et al. 1997). There, they encountered more archaic hominins: Neanderthals and, farther east, Denisovans. There was some intermixture. How much? Some have argued that modern Europeans and Asians are 3.4 to 7.9 percent admixed (Lohse and Frantz 2013). Most still opt for a lower figure of 1.5 to 2.1 percent (Prüfer et al. 2014).

But it wasn't only in Eurasia that modern humans encountered Neanderthal-like groups. Archaic hominins were present in Africa itself, some being relatively close to modern humans, and some more distantly related.

The latest DNA study has confirmed that modern humans intermixed with at least one archaic group as they expanded into western Africa:

The possible basal western African population lineage would represent the earliest known divergence of a modern human lineage that contributed a major proportion of ancestry to present-day humans. Such a lineage must have separated before the divergence of San ancestors, which is estimated to have begun on the order of 200-300 thousand years ago. (Skoglund et al. 2017)

This archaic ancestry is visible in human remains found at the Iwo Eleru rock shelter, in southwestern Nigeria, and dated to approximately 16,300 BP:

Our analysis indicates that Iwo Eleru possesses neurocranial morphology intermediate in shape between archaic hominins (Neanderthals and Homo erectus) and modern humans. This morphology is outside the range of modern human variability in the PCA and CVA analyses, and is most similar to that shown by LPA individuals from Africa and the early anatomically modern specimens from Skhul and Qafzeh. (Harvati et al., 2011)

Archaic ancestry is also visible in present-day West Africans, particularly in their teeth: 

[...] compared to other world populations, Africans south of the Sahara Desert are distinct dentally — especially in their expression of nine high- and two low-frequency morphological features. [...] the same nine high-frequency traits are also ubiquitous in the dentitions of extinct hominids and many extinct and extant non-human primates.  
[...] The presence and, indeed, prevalence (see next section), of high-frequency Sub-Saharan dental traits in fossil and recent hominoids—some of which are probably direct ancestors of modern humans, suggests they have been around for a long time.  
[...] A final ancestral feature found with some regularity in Sub-Saharan Africans, relative to other modern groups, is polydontia. Numerous cases of extra incisors, third premolars, and fourth molars have been noted [...] In one study (Watters, 1962) the incidence reached 2.5-3% in several hundred west Africans; many of the extra teeth were fully formed and erupted. "Typical" mammals exhibit three incisors and four premolars (Jordan et al., 1992). Polydontia is also found in living non-human primates. (Irish, 1998)

How much archaic ancestry do sub-Saharan Africans have today? The latest DNA study is silent on this point. Any answer can only be approximate, there being no reconstructed genome of this Neanderthal-like population. Moreover, there was probably more than one such population within Africa. Watson et al. (1997) attribute 13% of the sub-Saharan gene pool to a population that expanded some 111,000 years ago—when Skhul-Qafzeh hominins entered the Middle East from Africa. Those hominins were anatomically modern, or almost so, but culturally Neanderthal. Hammer et al. (2011) estimate that about 2% of the sub-Saharan African genome comes from a much more divergent population that split off from the ancestors of modern humans some 700,000 years ago. That admixture entered the sub-Saharan gene pool about 35,000 years ago, perhaps in Central Africa, since pygmy groups from that region have the most.

It looks like the proportion of archaic ancestry is higher in sub-Saharan Africans than in other modern humans. This is to be expected because of the broader range of archaic populations in Africa, including some that were almost modern anatomically and behaviorally. Admixture with them would have been likelier.

Admixture: good, bad, or neither?

Some alleles have successfully introgressed from archaic hominins, thus helping our ancestors adapt to new climates and new diets (Racimo et al. 2015). In general, however, we should not expect such alleles to perform as well in the body of a modern human as they did in the body of an archaic hominin. It's like taking a part from a Chevy and installing it on a Subaru. It might work, but I wouldn't count on it. 

If we look at Neanderthal admixture in the Eurasian genome, we see that natural selection has tended to remove functional genes, while leaving the non-functioning ones alone. 

Neanderthal ancestry decreases in proximity to functional elements in all populations [...] as does Denisovan ancestry in Oceanians [...] most likely reflecting greater selection against Neanderthal ancestry in low B statistic regions. Power to detect archaic ancestry is elevated close to regions of linked selection due to a reduction in the rates of incomplete lineage sorting caused by the lower effective population size in these regions, so these results are not artifacts of reduced power. Thus, similar processes appear to have worked to remove Neanderthal and Denisovan ancestry near genes. (Sankararaman et al. 2016)

Archaic admixture is also associated with reduced male fertility:

Our study provides new evidence in support of the hypothesis that reduced male fertility may be a common feature of admixture between human populations diverged by at least a half million years, a hypothesis that was previously suggested based on genetic patterns associated with the hybridization between Neanderthals and modern humans.

[...] One line of evidence for reduced fertility in male hybrids is that the proportion of archaic ancestry in modern humans is significantly reduced on chromosome X compared to the autosomes. This is suggestive of reduced male fertility as loci contributing to this phenotype are concentrated on chromosome X in hybrids of other species. We confirm an extreme reduction of Neanderthal ancestry on chromosome X (16%-34% of the autosomes depending on the population) and find a quantitatively similar reduction of Denisovan ancestry (21% of the autosomes in Oceanians).

The second line of evidence in support of the hypothesis of reduced fertility in hybrids is that there is a reduction of archaic ancestry in genes that are disproportionately expressed in testes, a known characteristic of male hybrid fertility (Sankararaman et al. 2016)

In sum, archaic admixture did provide modern humans with some ready-made alleles that have helped them adapt to new climates and new diets, but this advantage hardly applies to Africa. There, modern humans were already adapted to the local climate and diet. Archaic admixture couldn't have done much to help them adapt, since the new environments they faced were cultural ones of their own making.

References

Barbieri, C., A. Butthof, K. Bostoen, and B. Pakendorf. (2013). Genetic perspectives on the origin of clicks in Bantu languages from southwestern Zambia, European Journal of Human Genetics, 21(4), 430-436.
https://www.ncbi.nlm.nih.gov/pmc/articles/PMC3598317/  

Hammer, M.F., A.E. Woerner, F.L. Mendez, J.C. Watkins, and J.D. Wall. (2011). Genetic evidence for archaic admixture in Africa, Proceedings of the National Academy of Science (USA), 108(37), 15123-15128, www.pnas.org/cgi/doi/10.1073/pnas.1109300108

Harvati, K., C. Stringer, R. Grün, M. Aubert, P. Allsworth-Jones, C.A. Folorunso. (2011). The Later Stone Age Calvaria from Iwo Eleru, Nigeria: Morphology and Chronology. PLoS ONE 6(9): e24024. doi:10.1371/journal.pone.0024024
http://www.plosone.org/article/info%3Adoi%2F10.1371%2Fjournal.pone.0024024  

Irish, J.D. (1998). Ancestral dental traits in recent Sub-Saharan Africans and the origins of modern humans, Journal of Human Evolution, 34, 81-98.
http://www.sciencedirect.com/science/article/pii/S0047248497901913  

Lohse, K., and L.A.F. Frantz. (2013). Maximum likelihood evidence for Neandertal admixture in Eurasian populations from three genomes, Populations and Evolution, 1307, 8263
http://www.integratedbiology.com/uploads/2/5/6/9/25695765/_1307.8263.pdf  

Prüfer, K., F. Racimo, N. Patterson, F. Jay; et.al. (2014). The complete genome sequence of a Neandertal from the Altai Mountains, Nature, 505(7481), 43-49.
https://www.ncbi.nlm.nih.gov/pmc/articles/PMC4031459/

Racimo, F., S. Sankararaman, R. Nielsen, and E. Huerta-Sanchez. (2015). Evidence for archaic adaptive introgression in humans, Nature Reviews Genetics, 16(6), 359-371.
https://www.ncbi.nlm.nih.gov/pmc/articles/PMC4478293/  

Sankararaman, S., S. Mallick, N. Patterson, D, Reich; et al. (2016). The combined landscape of Denisovan and Neanderthal ancestry in present-day humans, Current Biology, 26(9), 1241-1247.
http://www.sciencedirect.com/science/article/pii/S0960982216302470  

Skoglund, P., J.C. Thompson, M.E. Prendergast, A. Mittnik; et al. (2017). Reconstructing prehistoric African population structure, Cell, 171(1), 59-71
http://www.cell.com/cell/fulltext/S0092-8674(17)31008-5  

Watson, E., P. Forster, M. Richards, and H-J. Bandelt. (1997). Mitochondrial footprints of human expansions in Africa, American Journal of Human Genetics, 61, 691-704.
https://ac.els-cdn.com/S000292970764333X/1-s2.0-S000292970764333X-main.pdf?_tid=9bebd320-a127-11e7-9e7c-00000aacb360&acdnat=1506257895_6658dfe089335953bd04987696fa7444  

Saturday, November 8, 2014

A look at an early European


Kostenki Man, reconstructed by Mikhail Gerasimov (1907-1970). An early European who was not yet phenotypically European.


Who were the first Europeans? We now have a better idea, thanks to a new paper about DNA from a man who lived some 38,700 to 36,200 years ago. His remains were found at Kostenki, a well-known Upper Paleolithic site in central European Russia (Seguin-Orlando et al., 2014).

Kostenki Man tells us several things about the first Europeans and, more broadly, the first non-African humans:

The Neanderthal encounter

Modern humans received their Neanderthal admixture when they were just spreading out of Africa some 54,000 years ago. At that time, they had not yet encountered the Neanderthals and were entering the territory of the Skhul/Qafzeh hominids, a semi-archaic people of the Middle East. So we may have got our Neanderthal admixture indirectly. The Skhul/Qafzeh hominids had probably interbred with their Neanderthal neighbors to the north, and our ancestors may have then picked up this admixture while in the Middle East. 

When our ancestors spread farther north into Europe, some 45,000 to 42,000 years ago, they could have interbred directly with Neanderthals, but they didn't. Perhaps the two groups were just too different. They seem to have intermixed only via a third party that was neither fully modern nor fully archaic.


A strange detour ... and then another!

There was initially a large continuous population across northern Eurasia, perhaps composed of nomads who pursued wandering herds of reindeer across the European Plain and its eastward extension into central and northern Asia.

Not long before the time of Kostenki Man, these Northern Eurasians began to split into three regional groups: Western Eurasians, Eastern Eurasians, and the ancestors of Middle Eastern farmers. The degree of reproductive isolation is unclear, however, and gene flow may have continued between all three groups until the onset of the last ice age some 25,000 years ago. This may be why Kostenki Man does not fit perfectly into any of the three groups, although he is genetically closest to Western Eurasians.

Yes, Northern Eurasians were ancestral to the early farming peoples of the Middle East. It seems that early modern humans had to head north, learn to hunt reindeer, and then head south again before they could start farming. Sounds like a strange detour. Wouldn't it have been easier to stay put and do it locally? You know, Middle-Eastern hunter-gatherers becoming Middle Eastern farmers? Apparently not.

It gets even more convoluted. After some of those Northern Eurasians had gone south to the Middle East, some of their farming descendants "returned" to Europe and partially replaced its hunter-gatherers, particularly in southern and central Europe. This second detour has been greeted with disbelief. Dienekes (2014), for instance, has written: "I don't think many archaeologists would derive European farmers from Russia (Russia is actually one of the last places in Europe that became agricultural)."

True, but farming requires a mindset that may have come from those northern hunters (Frost, 2014). When Piffer (2013) looked at human variation in alleles at COMT, a gene linked to executive function, working memory, and intelligence, he found that northern hunting peoples had more in common with farming peoples than with other hunter-gatherers, "possibly due to the higher pressure on technological skills and planning abilities posed by the adverse climatic conditions."

That mindset made farming possible, but the first steps toward farming could not be taken in a cold climate. They had to be taken in a place with a long growing season and a wide variety of domesticable plants and animals, such as in the Middle East. Once farming had developed there, it could move back north, while taking along its technologies, its food crops, and its livestock species. 

Farming can develop in the tropics with a "tropical" mindset, but it looks very different. The farming that arose in West Africa is overwhelmingly women's work and seems to have wholly developed out of female plant gathering. The guinea fowl is the only animal that has been domesticated for food consumption in sub-Saharan Africa.


The Ice Age was not so bad 

The Upper Paleolithic humans of northern and eastern Europe did not die out during the last ice age, as was commonly thought. They survived the glacial maximum intact.


The European phenotype came later

Kostenki Man was dark-skinned, dark-eyed, and rather short. These details, curiously enough, appear not in the paper but in a review of the paper, published by the same journal, as well as in an interview with one of the authors (Associated Press, 2014; Gibbons, 2014). 

So we now have an upper bound for the emergence of the European phenotype, i.e., light skin and a diverse palette of hair and eye colors. The lower bound has been set by the remains of a Swedish hunter-gatherer, dated to 8,000 years ago, who had the "European" allele for light skin at the gene SLC24A5 (Skoglund et al., 2014).


Conclusion

My main criticism centers on the dating to 38,700 - 36,200 years ago. At the Kostenki site, the radiocarbon dating used to be some 10,000 years younger. It was then recalibrated to an older range of dates when a layer of volcanic ash at the site was attributed to a volcano that had erupted in southern Italy some 39,000 years ago. This recalibration was initially controversial, but the controversy has since subsided (Sinitsyn and Hoffecker, 2006). I would not rule out a subsequent re-recalibration.

By retrieving ancient DNA from an early modern human, we have made a key advance in human paleogenetics, perhaps more so than by sequencing the Neanderthal genome. We again see that evolution did not slow down with the emergence of anatomically and behaviorally modern humans some 60,000 years ago. It actually began to speed up, as humans began to enter not only new natural environments but also new cultural environments of their own making.
 

References 

Associated Press (2014). DNA study dates Eurasian split from East Asians, The Columbus Dispatch, November 6
http://hosted2.ap.org/OHCOL/07e34bb59e064cedb7e2776e8db4b4f7/Article_2014-11-06-EU--Eurasian%20Split/id-ae36fa368c634c7383d807942bd5fe67 

Dienekes (2014). Genome of Kostenki-14, an Upper Paleolithic European (Seguin-Orlando, Korneliussen, Sikora, et al. 2014), Dienekes' Anthropology Blog, November 7
http://dienekes.blogspot.ca/2014/11/genome-of-kostenki-14-upper-paleolithic.html  

Frost, P. (2014). The first industrial revolution, Evo and Proud, January 18
http://evoandproud.blogspot.ca/2014/01/the-first-industrial-revolution.html 

Gibbons, A. (2014). European genetic identity may stretch back 36,000 years, Science, News, November 6
http://news.sciencemag.org/archaeology/2014/11/european-genetic-identity-may-stretch-back-36000-years 

Piffer, D. (2013). Correlation of the COMT Val158Met polymorphism with latitude and a hunter-gather lifestyle suggests culture-gene coevolution and selective pressure on cognition genes due to climate, Anthropological Science, 121, 161-171.
https://lesacreduprintemps19.files.wordpress.com/2014/01/correlation-of-the-comt-val158met-polymorphism-with-latitude-and-a-hunter-gather-lifestyle-suggests-culturee28093gene-coevolution-and-selective-pressure-on-cognition-genes-due-to-climate.pdf 

Seguin-Orlando, A., T.S. Korneliussen, M. Sikora, A.-S. Malaspinas, A. Manica, I. Moltke, A. Albrechtsen, A. Ko, A. Margaryan, V. Moiseyev, T. Goebel, M. Westaway, D. Lambert, V. Khartanovich, J.D. Wall, P.R. Nigst, R.A. Foley, M.M. Lahr, R. Nielsen, L. Orlando, and E. Willerslev. (2014). Genomic structure in Europeans dating back at least 36,200 years, Science, Published online 6 November 2014
http://www.sciencemag.org/content/early/2014/11/05/science.aaa0114
http://www2.zoo.cam.ac.uk/manica/ms/2014_Seguin_Orlando_et_al_Science.pdf  

Sinitsyn, A.A., and J.F. Hoffecker. (2006). Radiocarbon dating and chronology of the Early Upper Paleolithic at Kostenki, Quaternary International, 152-153, 164-174.
http://www.sciencedirect.com/science/article/pii/S1040618206000206 

Skoglund, P., H. Malmstrom, A. Omrak, M. Raghavan, C. Valdiosera, T. Gunther, P. Hall, K. Tambets, J. Parik, K-G. Sjogren, J. Apel, E. Willersley, J. Stora, A. Gotherstrom, and M. Jakobsson. (2014). Genomic diversity and admixture differs for stone-age Scandinavian foragers and farmers, Science, 344 (6185), 747-750.
http://www.sciencemag.org/content/344/6185/747.short
 

Saturday, October 4, 2014

Making the big time ... elsewhere


Skull from Broken Hill (Kabwe), Zambia. This kind of human was still around when the Neanderthals were going extinct in Europe. (Wikicommons)


East Africa, 60,000 to 80,000 years ago. The relative stasis of early humans was being shaken by a series of population expansions. The last one went global, spreading out of Africa, into Eurasia and, eventually, throughout the whole world (Watson et al., 1997). Those humans became us.

This expansion took place at the expense of more archaic humans: Neanderthals in Europe, the Middle East, and Central Asia; Denisovans in East Asia; and mysterious hobbit-like creatures in parts of Southeast Asia.

And in Africa itself? We know less about those archaic humans, partly because the archeological record is so patchy and partly because ancient DNA does not survive as long in the tropics. Over time, the double helix breaks down, and this decomposition occurs faster at higher ambient temperatures. We'll probably never be able to reconstruct the genome of archaic Africans.

Yet they did exist. Surprisingly, they held out longer in parts of Africa than their counterparts did much farther away. A Nigerian site has yielded a skull that is only about 16,300 years old and yet looks intermediate in shape between modern humans on the one hand and Neanderthals and Homo erectus on the other. It resembles the skull of a very early modern human, like the ones who once lived at Skhul and Qafzeh in Israel some 80,000 to 100,000 years ago (Harvati et al., 2011; Stojanowski, 2014).

Archaic humans also held out in southern Africa. The Broken Hill or Kabwe skull, from Zambia has been dated to 110,000 years ago and looks very much like a Homo erectus (Bada et al., 1974; Stringer, 2011). This pre-sapiens human seems to have lasted into much later times. Hammer et al. (2011) found that about 2% of the current African gene pool comes from a population that split from ancestral modern humans some 700,000 years ago. They dated the absorption of this archaic DNA to about 35,000 years ago and placed it in Central Africa, since the level of intermixture is highest in pygmy groups from that region.
 

Cognitive modernity: less awesome on its home turf

Why did archaic humans survive longer in Africa than elsewhere? Some of them were more advanced than the Neanderthals or Denisovans, and perhaps better able to fend off invasive groups. This was the case with archaic West Africans, who seem to have been transitional between pre-sapiens and sapiens. They may have met modern humans on a more level playing field while enjoying the home team advantage.

On the other hand, archaic southern Africans look clearly pre-sapiens. What was levelling their playing field? Perhaps modern humans had advantages that were more useful outside Africa. Klein (1995) has argued that this advantage was cognitive, specifically a superior ability not only to create ideas but also to share them with other individuals via language—in a word, culture. This cognitive edge may have been more useful outside the tropics, where the yearly cycle forced humans to plan ahead collectively and keep warm collectively by building shelters and making garments. The result was a much wider range of human technology: deep storage pits for meat refrigeration; hand-powered rotary tools; kilns for ceramic manufacture; woven textiles; eyed sewing needles; traps and snares; and so on (Frost, 2014).

Modern humans were thus pre-adapted in Africa for later success elsewhere. We see this in their rapid penetration of cold environments unlike anything in their place of origin. By 43,500 years ago, they were already present in Central Europe at a time when it was barren steppe with some boreal forest in sheltered valleys (Nigst et al., 2014).

Pre-adaptation is a recurring oddity of evolution. A new ability may initially be a bit helpful and only later truly awesome. Does this mean that evolution anticipates future success? Well, no. It's just that the difference between failure and success—or between so-so success and the howling kind—often hinges on a few things that may or may not exist in your current environment. By moving to other environments, you increase your chances of finding one that will put your talents to better use. Success is fragile, but so is failure.
 

References 

Bada, J.L., R.A. Schroeder, R. Protsch, & R. Berger. (1974). Concordance of Collagen-Based Radiocarbon and Aspartic-Acid Racemization Ages, Proceedings of the National Academy of Sciences (USA), 71, 914-917.
http://www.pnas.org/content/71/3/914.short 

Frost, P. (2014). The first industrial revolution, Evo and Proud, January 18
http://evoandproud.blogspot.ca/2014/01/the-first-industrial-revolution.html

Hammer, M.F., A.E. Woerner, F.L. Mendez, J.C. Watkins, and J.D. Wall. (2011). Genetic evidence for archaic admixture in Africa, Proceedings of the National Academy of Sciences (USA), 108, 15123-15128.

Harvati, K., C. Stringer, R. Grün, M. Aubert, P. Allsworth-Jones, C.A. Folorunso. (2011). The Later Stone Age Calvaria from Iwo Eleru, Nigeria: Morphology and Chronology. PLoS ONE 6(9): e24024. doi:10.1371/journal.pone.0024024
http://www.plosone.org/article/info%3Adoi%2F10.1371%2Fjournal.pone.0024024 

Klein, R.G. (1995). Anatomy, behavior, and modern human origins, Journal of World Prehistory, 9, 167-198.
http://link.springer.com/article/10.1007/BF02221838 

Nigst, P.R., P. Haesaerts, F. Damblon, C. Frank-Fellner, C. Mallol, B. Viola, M. Gotzinger, L. Niven, G. Trnka, and J-J. Hublin. (2014). Early modern human settlement of Europe north of the Alps occurred 43,500 years ago in a cold steppe-type environment, Proceedings of the National Academy of Sciences (USA), published online before print
http://www.pnas.org/content/early/2014/09/16/1412201111.short 

Stojanowski, C.M. (2014). Iwo Eleru's place among Late Pleistocene and Early Holocene populations of North and East Africa, Journal of Human Evolution, epub ahead of print
http://www.sciencedirect.com/science/article/pii/S0047248414000876 

Stringer, C. (2011). The chronological and evolutionary position of the Broken Hill cranium. American Journal of Physical Anthropology, 144(supp. 52), 287

Watson, E., P. Forster, M. Richards, and H-J. Bandelt. (1997). Mitochondrial footprints of human expansions in Africa, American Journal of Human Genetics, 61, 691-704. 0024024
http://www.plosone.org/article/info%3Adoi%2F10.1371%2Fjournal.pone.0024024