Showing posts with label Phil Rushton. Show all posts

Saturday, July 11, 2020

Did women jumpstart recent cognitive evolution?


Scatter plots of frequencies of CASC5 variants by sex (Shi et al. 2017). During the last ice age, natural selection favored an increase in the gray matter of ancestral East Asians ... primarily in women.


Back in 2005 there was much interest in genes that regulate brain size, particularly in the ways they varied geographically within our species. It was found that two of these genes, Microcephalin and ASPM, continued to evolve as modern humans spread out of Africa. The latest variant of Microcephalin arose some 37,000 years ago in Eurasia and is still largely confined to the indigenous peoples of Eurasia and the Americas (Mekel-Bobrov et al. 2005). The latest variant of ASPM appeared even later, some 5,800 years in the Middle East (Evans et al. 2005).

Interest fell off when no association could be shown between the new variants and IQ or brain size (Mekel-Bobrov et al. 2007; Rushton et al. 2007; see also Frost 2020). Since then, we have learned that the new ASPM variant is associated with a larger cerebral cortex, and not a larger brain as a whole. Overall brain volume seems to be constrained in modern humans, perhaps by the breadth of a woman's pelvis during childbirth or simply by the high metabolic costs of brain tissue (Ali and Meier 2008; Frost 2020). As for the lack of an association with IQ, we now know that IQ correlates poorly or not at all with some cognitive abilities, like executive function and face recognition.

But what do the new variants actually do? Perhaps a specialized mental task.  It has been suggested that the new ASPM variant assists the brain in processing non-tonal language or alphabetical script (Dediu and Ladd 2007; Frost 2007).


CASC5, another gene for brain growth

Interest has since grown in another gene that regulates brain growth, CASC5. Like Microcephalin and ASPM, it has undergone recent evolution in the modern human lineage:

[...] the CASC5 gene contains mutations in modern humans, but not in Denisovans (Meyer et al. 2012) and this gene also shows distinct sequence divergence between modern humans and Neanderthals (Prufer et al. 2014). These data suggest that CASC5 is an important gene for human neurogenesis, and may harbor modern human specific mutations contributing to the recent evolutionary change of the human brain. (Shi et al. 2017)

Shi et al. (2017) found evidence of recent evolutionary change. Specifically, two nucleotides of CASC5 have been replaced with a new variant in all modern humans. Six other nucleotides have become polymorphic, with some people having the new variants and others not. These polymorphisms show regional differences:

- In four of the polymorphisms, the new variant has a much higher frequency in East Asians than in Europeans or Africans.
- In one polymorphism, it has a much higher frequency in Europeans than in the other two regional groups.
- The remaining polymorphism shows no differences in frequency between the three regional groups.

By and large, the new variants have been under strong positive selection, particularly among East Asians. When the authors examined the six polymorphisms, they found signals of selection for five of them in East Asians and for one in Europeans.


The new variants and brain characteristics

The authors then looked for correlations between the new variants and certain characteristics of the brain, specifically total brain volume, gray matter volume, and white matter volume. To this end, 267 healthy participants were recruited for brain imaging (Han Chinese, 178 females and 89 males, mean age 35.4 ± 12.5 years). All of them were free from mental disorders, drug abuse, alcohol dependence, and brain injury.

Gray matter was significantly larger in participants with the new variant than in those with the ancestral variant at five of the nucleotide sites, including the four polymorphic ones—the same ones that showed differences in variant frequency between East Asians and Europeans. When the authors examined the one polymorphism whose variants were equally common in East Asians, Europeans, and Africans, they found no brain differences between participants with the new variant and those with the ancestral one.

When the authors broke their data down by sex, they found that the new variants were significantly associated with a higher volume of gray matter only in women, not in men, although men seemed to trend in the same direction. The authors suggest that this effect would be significant in men if the number of male participants were larger. Probably. But it seems to me there would still be a sex difference, the number of participants being already large enough.


Ice age origin of the new variants

The authors say the new variants became prevalent "after modern humans migrated out of Africa less than 100,000 years ago." We can narrow down the time range further. The new variants are also present at high frequencies among the indigenous peoples of North and South America; therefore, they must have become prevalent before ancestral Amerindians crossed into North America some 12,000 years ago, apparently in a population that was ancestral both to Amerindians and to East Asians. That would be long before the time of recorded history and even before the Holocene, at a time when northern Eurasia was experiencing glacial conditions.

Did those conditions select for cognitive ability? Cold, seasonal environments did impose new cognitive demands on early modern humans, first by increasing their need to plan ahead over a yearly cycle and second by providing them with new tasks: garment making, needlework, weaving, leatherworking, and kiln operation. Women performed those tasks because the environment offered them few opportunities for food gathering—the usual female activity before the advent of farming. They thus moved into artisanal tasks that not only required greater cognitive ability but also offered much potential for further development. This was the "original industrial revolution" and it was led by women (Frost 2019a).

We can better understand this sexual division of labor by studying northern hunter-gatherers of recent times. According to a cross-cultural study, if women are less involved in food gathering, they specialize in activities unrelated to food procurement, i.e., house building, leatherworking, and burden carrying (Waguespack 2005). A study of two Inuit groups found the highest degree of technological complexity in garment making and shelter building, both of which are wholly or largely women's work (Oswalt 1976). Cold environments thus change the sexual division of labor among hunter-gatherers in a crucial way: while men continue to be food providers, women develop new technologies.

These findings may explain the recent evolution of CASC5: women were the focus of selection for cognitive ability during Ice Age times. But why was the selection stronger among ancestral East Asians than among ancestral Europeans? It looks like the climate at that time was more severe in northern Asia than in northern Europe. Europe benefited from the moderating influence of the Atlantic, which made for a milder and moister climate. Conditions were much colder and drier in northern Asia.

The evolution of human intelligence cannot be reduced to a single unified theory. Cold environments emancipated women from the mental straitjacket of food gathering, thus putting humans on the path to social complexity. That path, however, would take them to latitudes farther south in temperate and even tropical environments where they would be exposed to new cognitive demands. With the end of hunting, men moved not only into farming but also into the artisanal activities that women had developed. The same period saw a decline in brain volume that was greater in women than in men—an indication that cognitive demands were particularly high before the Holocene, and even more so for women (Frost 2019b).

The Holocene thus saw northern populations expand southward and eventually cover almost all of Eurasia, North Africa, Oceania, and the Americas. Those populations had a cognitive advantage that made them better able to exploit the social complexity emerging farther south. This point was made by Darwin's colleague Alfred Russel Wallace:

So when a glacial epoch comes on, some animals must acquire warmer fur, or a covering of fat, or else die of cold. Those best clothed by nature are, therefore, preserved by natural selection. Man, under the same circumstances, will make himself warmer clothing, and build better houses; and the necessity of doing this will react upon his mental organisation and social condition [...] a hardier, a more provident, and a more social race would be developed, than in those regions where the earth produces a perennial supply of vegetable food, and where neither foresight nor ingenuity are required to prepare for the rigours of winter. And is it not the fact that in all ages, and in every quarter of the globe, the inhabitants of temperate have been superior to those of tropical countries? All the great invasions and displacements of races have been from North to South, rather than the reverse.


References

Ali, F. and R. Meier. (2008). Positive selection in ASPM is correlated with cerebral cortex evolution across primates but not with whole brain size. Molecular Biology and Evolution 25(11): 2247-2250.

Dediu, D., and R. Ladd. (2007). Linguistic tone is related to the population frequency of the adaptive haplogroups of two brain size genes, ASPM and Microcephalin. Proceedings of the National Academy of Sciences 104(26): 10944-10949

Evans, P. D., Gilbert, S. L., Mekel-Bobrov, N., Vallender, E. J., Anderson, J. R., Vaez-Azizi, L. M., et al. (2005). Microcephalin, a gene regulating brain size, continues to evolve adaptively in humans. Science 309: 1717-1720.

Frost, P. (2007). The spread of alphabetical writing may have favored the latest variant of the ASPM gene. Medical Hypotheses 70: 17-20.

Frost, P. (2019a). The Original Industrial Revolution. Did Cold Winters Select for Cognitive Ability? Psych 1(1): 166-181

Frost, P. (2019b). Why did brain size decrease after the ice age? Evo and Proud, July 6

Frost, P. (2020). A second look at ASPM. Evo and Proud, April 14

Mekel-Bobrov, N., S.L. Gilbert, P.D. Evans, E.J. Vallender, J.R. Anderson, R.R. Hudson, S.A. Tishkoff and B.T. Lahn. (2005). Ongoing adaptive evolution of ASPM, a brain size determinant in Homo sapiens. Science 309: 1720-1722

Mekel-Bobrov, N., D. Posthuma, S.L. Gilbert, P. Lind, M.F. Gosso, et al. (2007). The ongoing adaptive evolution of ASPM and Microcephalin is not explained by increased intelligence. Human Molecular Genetics 16(6): 600-608.

Oswalt, W.H. (1976). An Anthropological Analysis of Food-Getting Technology, 1st ed.; John Wiley and Sons: New York, NY, USA.

Rushton, J.P., P.A. Vernon, and T.A. Bons. (2007). No evidence that polymorphisms of brain regulator genes Microcephalin and ASPM are associated with general mental ability, head circumference or altruism. Biology Letters-UK 3(2): 157-60.

Shi, L., Hu, E., Wang, Z. et al. (2017). Regional selection of the brain size regulating gene CASC5 provides new insight into human brain evolution. Human Genetics 136: 193-204. https://doi.org/10.1007/s00439-016-1748-5

Waguespack, N.M. (2005). The organization of male and female labor in foraging societies: Implications for early Paleoindian archaeology. American Anthropologist 107: 666-676.

Wallace, A.R. (1864). The Origin of Human Races and the Antiquity of Man deduced from the Theory of "Natural Selection." Journal of the Anthropological Society of London, 2, clviii-clxxxvii, Alfred Russel Wallace Classic Writings. Paper 6. http://digitalcommons.wku.edu/dlps_fac_arw/6


Friday, June 19, 2020

Cleansing the scientific literature ... again


J. Philippe Rushton (Wikicommons). Eight years later, one of his studies is being “removed” from the scientific literature.


Seven years ago I wrote about Danish psychologist Helmuth Nyborg and the attempts to "unpublish" a study he had already published. At first thought, the idea seemed strange to me:

I was initially stumped by the ruling that Dr. Nyborg must withdraw his study from the scientific literature. How can one withdraw an already published study? Then the penny dropped. Most journals are now published online, and cash-strapped university libraries have been phasing out their paper subscriptions. (Frost 2013)

I and many others complained to the Danish minister responsible for that decision, and it was reversed.

Now, the same thing is happening again, in the heart of the Free World:

An article claiming that skin pigmentation is related to aggression and sexuality in humans will be retracted, Elsevier announced today. The study, "Do pigmentation and the melanocortin system modulate aggression and sexuality in humans as they do in other animals?" was published online in Personality and Individual Differences, an Elsevier journal, on March 15, 2012. The study's authors, John Rushton and Donald Templer, both deceased, hypothesized that skin color was related to aggression and sexuality in humans. It has been cited just nine times in eight years, according to Clarivate Analytics' Web of Science. (Retraction Watch 2020)

According to Google Scholar it has been cited fifteen times. Anyway, a study’s worthiness isn't decided by a show of hands, either now or in the future. Opinions change, and fringe science may eventually become mainstream. Or vice versa.

That brings me to another point. For eight years that study was legitimate. Now, it no longer is. Thanks to George Floyd.

Actually, his death was only a pretext. The mob feels no differently today than it did before May 25. What has changed is its ability to get what it wants ... with no pushback. Let’s not kid ourselves. This is a power grab by people who already have much power over the most important aspect of human culture—the flow of information. If you control a few chokepoints, you can get most people to believe almost anything.

“Power” may not be the right word. The aim is not simply to control institutions but rather to control how we perceive and understand reality. These are people who believe that ideas matter, and they want control over ideas, even in the scientific literature (!).

I don't wish to judge whether Rushton and Templer were "right." Once a study has passed peer review and been published, that judgement belongs solely to the reader. Personally, I feel they were right in some respects and wrong in others. They were right to argue that darker-colored animals tend to be larger and more aggressive, this being true not only between species but also within species:

Ducrest et al. (2008) reviewed data on over 40 wild vertebrate species showing that within each species, darker pigmented individuals averaged higher levels of aggression and sexual activity than lighter pigmented individuals, with a larger body mass, more resistance to stress, and greater physical activity when grooming. The relationship between coloring and behavioral dominance was robust across three species of mammal (African lion, soay sheep, and white-tailed deer), four species of fish (mosquito fish, guppy, green swordtail, and Arctic charr), four species of reptile (asp viper, adder, fence lizard, and spiny lizard), one amphibian species (spadefoot toad) and 36 species of bird.

In captive Hermann's tortoises (Eurotestudo boettgeri), another reptile species, Mafli, Wakamatsu, and Roulin (2011) found darker shell coloration predicted greater aggressiveness and boldness. Darker individuals were more aggressive in male-male confrontations and bolder towards humans, independent of body size and ambient temperature. (Melanin based color traits are a criterion in mate choice.)

Validation of the pigmentation system as causal to the naturalistic observations was demonstrated by experimentally manipulating pharmacological dosages and by studies of cross-fostering (Ducrest et al., 2008). Thus, melanocortin hormone levels predicted the amount of testosterone and other sexual steroids along with concomitant increases (or decreases) in aggression and sexual behavior. Placing darker versus lighter pigmented individuals with adoptive parents of the opposite pigmentation did not modify offspring behavior. (Rushton and Templer 2012)

Yes, melanin does correlate with aggressiveness, especially male aggressiveness. Unlike Rushton and Templer, however, I don't believe the correlation is causal, at least not wholly. It probably began as an accidental association: newborns are generally less pigmented, and this has resulted in a mental association of lightness with weakness and immaturity. Conversely, darkness is associated with strength and maturity. The age difference in pigmentation has been amplified by sexual selection in many species, particularly polygynous species where males have to compete against each other for access to females

We humans make the same mental association, particularly darker-skinned humans. Among them, the contrast between infant and adult pigmentation is striking:

There is a rather widespread concept in Black Africa, according to which human beings, before "coming" into this world, dwell in heaven, where they are white. For, heaven itself is white and all the beings dwelling there are also white. Therefore the whiter a child is at birth, the more splendid it is. In other words, at that particular moment in a person's life, special importance is attached to the whiteness of his colour, which is endowed with exceptional qualities.

According to the same concept, it is also claimed that a newborn baby is not only white but also a soft being during the time between his birth and his acceptance into the society. Furthermore, during this entire period, he is not considered a real person, and this may go so far that parents and society may do away with him at will for reasons that are peculiar to each social group. Having been done away with, these beings are considered to return automatically to the place where they came from, that is, to heaven. (Zahan 1974, pp. 385-387)

This mental association may have become a factor in the struggle by men for mates. In highly polygynous societies, such as those of sub-Saharan Africa, darker-skinned men would be seen as more masculine, and threatening, by other men ... and by women.  Among human populations, darkness of skin correlates significantly with the polygyny rate, even after adjusting for latitudinal variation in skin color (Manning et al. 2004). It looks like selection has favored a darker color in adult males, particularly in a context of intra-male rivalry for mates, and this selection has probably occurred in many species.

I may be wrong. Perhaps Rushton and Templer were wrong. Perhaps nobody knows the truth on this point. That's why we don't unpublish scientific studies. No one has the last word in intellectual debate, and that's how things should be.

Elsevier is aware of the taboo it's treading on:

It is a general principle of scholarly communication that the editor of a learned journal is solely and independently responsible for deciding which articles submitted to the journal shall be published. In making this decision the editor is guided by policies of the journal's editorial board and constrained by such legal requirements in force regarding libel, copyright infringement and plagiarism.  An outcome of this principle is the importance of the scholarly archive as a permanent, historic record of the transactions of scholarship. Articles that have been published shall remain extant, exact and unaltered as far as is possible. However, very occasionally circumstances may arise where an article is published that must later be retracted or even removed. (Elsevier 2020)

Until now, unpublishing wasn’t even “very occasional.” I know of a few cases where a paper was retracted shortly after publication. But eight years after? That just wasn’t done. Now it’s been done. The taboo has been broken, and we're going to see more and more "removals."


References

Elsevier (2020). Article withdrawal. https://www.elsevier.com/about/policies/article-withdrawal

Frost, P. (2012). Dark coloration and male aggressiveness: Is there a link? Evo and Proud, March 31
https://evoandproud.blogspot.com/2012/03/dark-coloration-and-male-aggressiveness.html

Frost, P. (2013). Cleansing the scientific literature. Evo and Proud, November 23
http://evoandproud.blogspot.com/2013/11/cleansing-scientific-literature.html

Manning, J.T., P.E. Bundred, and F.M. Mather. (2004). Second to fourth digit ratio, sexual selection, and skin colour. Evolution and Human Behavior 25(1): 38-50.
https://doi.org/10.1016/s1090-5138(03)00082-5

Retraction Watch. (2020). Elsevier journal to retract 2012 paper widely derided as racist. June 17 https://retractionwatch.com/2020/06/17/elsevier-journal-to-retract-2012-paper-widely-derided-as-racist/

Rushton, J. P., and D.I. Templer. (2012). Do pigmentation and the melanocortin system modulate aggression and sexuality in humans as they do in other animals? Personality and Individual Differences 53(1): 4-8
https://www.sciencedirect.com/science/article/pii/S0191886912000840 

Zahan, D. (1974). White, Red and Black: Colour Symbolism in Black Africa. In A. Portmann and R. Ritsema (Eds.) The Realms of Colour, Eranos 41 (1972): 365-395, Leiden: Eranos.
https://doi.org/10.2307/1573594

Tuesday, April 14, 2020

A second look at ASPM


Worldwide frequency of the new ASPM variant (Mekel-Bobrov et al. 2007)


Fifteen years ago, Science published a major finding: the human brain was still evolving well after the dawn of history. This could be seen in the evolution of ASPM, a gene that severely reduces brain size if it fails to function during development.

Here, we show that one genetic variant of ASPM in humans arose merely about 5800 years ago and has since swept to high frequency under strong positive selection. These findings, especially the remarkably young age of the positively selected variant, suggest that the human brain is still undergoing rapid adaptive evolution. (Mekel-Bobrov et al. 2007)

This variant seems to have come from the Middle East, where it is most prevalent today (37-52%). Its prevalence is next highest in Europe (38-50%). It is much less common in East Asia (0-25%) and virtually absent almost everywhere else.

Interest waned in the subject when several researchers found no association between the new variant and IQ scores or brain size (Mekel-Bobrov et al. 2007; Rushton et al. 2007). At the time it was widely thought, notably by J. Philippe Rushton, that IQ covers all aspects of mental effort. When I asked him whether the researchers had measured mental endurance, he replied: "No, they just used the standard IQ tests, head circumference, and (in our case) a test of altruism. [...] Generally there isn't thought to be much left to be explained after g is taken out."

This view has since been called into question. Some cognitive abilities correlate poorly with IQ, like executive function (Arffa 2007). Others show no correlation at all, like face recognition (Zhu et al. 2010). Furthermore, there has been growing evidence that the different ASPM variants of modern humans affect only some parts of the brain, and not the entire brain. According to a comparative study of primate species, the evolution of ASPM does not correlate with major changes in the whole brain or in cerebellum size: 

Particularly striking is the result that only major changes of cerebral cortex size and not major changes in whole brain or cerebellum size are associated with positive selection in ASPM. This is consistent with an expression report indicating that ASPM's expression is limited to the cerebral cortex of the brain (Bond et al. 2002). Our findings stand in contrast to recent null findings correlating ASPM genotypes with human brain size variation. Those studies used the relatively imprecise phenotypic trait of whole brain instead of cerebral cortex size (Rushton, Vernon, and Bons 2006; Woods et al. 2006; Thimpson et al. 2007). Although previous studies have shown that parts of the brain scale strongly with one another and especially with whole brain (e.g., Finlay and Darlington 1995), evidence here suggests that different brain parts still have their own evolutionary and functional differentiation with unique genetic bases. (Ali and Meier 2008)

Another comparative study found that ASPM had undergone accelerated change in chimpanzee, bonobo, and human lineages. Perhaps more interestingly, the effects were confined to development of the cerebral cortex:

Our findings indicate that ASPM variation is potentially associated with cerebral ventricular volume in chimpanzees, but not with any of the other brain structure measures. Ventricles are a critical site of neuronal proliferation in early development. Furthermore, the cerebrospinal fluid which circulates through the ventricles throughout life carries proteins that play important roles in central nervous system development and maintenance, like Sonic Hedgehog protein and Insulin-like Growth Factor 2.

Sonic Hedgehog protein?

Thus, variation in ventricular volume may affect the circulation of growth factors that could potentially influence the regulation of cerebral cortical development. Alternatively, because ASPM has a significant effect on neural progenitor cycling along the ventricles in fetal life, the association shown in our study may be a result of how brain size is patterned by ASPM during neurogenesis in early development. It has been shown that ASPM plays a role in regulating the affinity of ventricular radial glial cells (VRGs) for the ventricular surface. (Singh et al. 2019)

While there is also a broader role in brain development and brain size, it is usually limited to extreme cases, like microcephaly:

The abundance of ASPM mutations in human patients with microcephaly suggests that the gene plays a significant role in the regulation of brain size; however, variation in the gene has not always shown direct impact on brain circumference, volume, and intelligence in non-pathological populations. It is possible that ASPM interacts with other genes to affect brain volume, and thus associations depend on genetic background. Furthermore, selective pressure on ASPM may be associated with other aspects of neuronal function that do not lead to overt changes in brain structure, or might have a pleiotropic effect in other areas of the body, as ASPM is also expressed outside of the brain (Singh et al. 2019)


Possible explanations for the new ASPM variant

Shift from tonal to nontonal language?

So what made the new ASPM variant so successful? Two British researchers, Dan Dediu and D. Robert Ladd argue that it was a shift from tonal to non-tonal language. After showing that nontonality correlates geographically with the new ASPM variant (and also a new variant of the Microcephalin gene), they note that "the fact that nontonality is associated with the derived haplogroups suggests that tone is phylogenetically older and that the bias favors nontonality" (Dediu Ladd 2007).

If this is true, tonality gave way to nontonality in the Middle East when the new ASPM variant arose there some six thousand years ago. Yet we have no evidence of such a shift. Furthermore, languages have usually evolved from nontonality to tonality: "it seems to be the dominant view in the literature that tones arose from a toneless state" (Abramson 2004).

Spread of alphabetical writing?

I have argued for another explanation: the new ASPM variant was successful because it somehow assisted a mental task that originated in the Middle East some six thousand years ago and then spread into Europe. The task was alphabetical writing, specifically the mental process of transcribing speech and copying texts into alphabetical characters. Though more easily learned than ideographs, these characters place higher demands on the mind, especially under premodern conditions (continuous text with little or no punctuation, real-time stenography, absence of automated assistance for publishing or copying, etc.). This task was largely assigned to scribes of various sorts who enjoyed privileged status and probably superior reproductive success, thereby spreading the new ASPM variant throughout the population (Frost 2007).


Conclusion

For a brief time, over a decade ago, it seemed we had hard evidence that the human brain was still evolving during the time of recorded history. That evidence was soon rejected and largely forgotten, ironically through the efforts of J. Philippe Rushton. It didn't fit his model. As he saw it, if something fails to correlate with IQ, specifically with the g factor, it cannot be a cognitive ability and is unworthy of interest. 

Rushton was also held back by the idea that human evolution had largely ended with the end of the last ice age. Though intrigued by the contrary idea of ongoing human evolution, he never brought it into his theoretical work and generally treated it like an unwanted strip of film on a cutting-room floor.


References

Abramson, A.S. (2004). The plausibility of phonetic explanations of tonogenesis. In: Fant, G., Fujisaki, H., Cao, J., Xu, Y. (Eds.), From traditional phonology to modern speech processing: Festschrift for Professor Wu Zongji's 95th birthday. Beijing: Foreign Language Teaching and Research Press, 17-29.
http://www.haskins.yale.edu/Reprints/HL1336.pdf

Ali, F. and R. Meier. (2008). Positive selection in ASPM is correlated with cerebral cortex evolution across primates but not with whole brain size. Molecular Biology and Evolution 25(11): 2247-2250.
http://www.haskins.yale.edu/Reprints/HL1336.pdf

Arffa, S. (2007). The relationship of intelligence to executive function and non-executive function measures in a sample of average, above average, and gifted youth. Archives of Clinical Neuropsychology 22(8): 969-978
https://academic.oup.com/acn/article/22/8/969/3025 

Dediu, D., and R. Ladd. (2007). Linguistic tone is related to the population frequency of the adaptive haplogroups of two brain size genes, ASPM and Microcephalin. Proceedings of the National Academy of Sciences 104(26):10944-10949
https://langev.com/pdf/dediu07linguisticTonePNAS.pdf

Frost, P. (2007). The spread of alphabetical writing may have favored the latest variant of the ASPM gene. Medical Hypotheses 70: 17-20.
http://www.sciencedirect.com/science/article/pii/S0306987707003234

Frost, P. (2008). Decoding the ASPM puzzle. Evo and Proud, August 27
http://evoandproud.blogspot.com/2008/08/decoding-aspm-puzzle.html  

Mekel-Bobrov, N., S.L. Gilbert, P.D. Evans, E.J. Vallender, J.R. Anderson, R.R. Hudson, S.A. Tishkoff and B.T. Lahn. (2005). Ongoing adaptive evolution of ASPM, a brain size determinant in Homo sapiens. Science 309: 1720-1722
https://www.researchgate.net/publication/7611130_Ongoing_Adaptive_Evolution_of_ASPM_a_Brain_Size_Determinant_in_Homo_Sapiens  
Mekel-Bobrov, N., D. Posthuma, S.L. Gilbert, P. Lind, M.F. Gosso, et al. (2007). The ongoing adaptive evolution of ASPM and Microcephalin is not explained by increased intelligence. Human Molecular Genetics 16(6): 600-608.
https://academic.oup.com/hmg/article/16/6/600/610971

Rushton, J.P., P.A. Vernon, and T.A. Bons. (2007). No evidence that polymorphisms of brain regulator genes Microcephalin and ASPM are associated with general mental ability, head circumference or altruism. Biology Letters-UK 3(2):157-60.
https://royalsocietypublishing.org/doi/full/10.1098/rsbl.2006.0586 

Singh, S.V., N. Staes, E.E. Guevara, S.J. Schapiro, J.J. Ely, et al. (2019). Evolution of ASPM coding variation in apes and associations with brain structure in chimpanzees. Genes, Brain and Behavior 18:e12582.
https://dukespace.lib.duke.edu/dspace/bitstream/handle/10161/19252/Singh_etal2019.pdf?sequence=2

Zhang, J. (2003). Evolution of the Human ASPM Gene, a Major Determinant of Brain Size. Genetics 165(4): 2063-2070.
https://www.genetics.org/content/165/4/2063.short

Zhu, Q., Y. Song, S. Hu, X. Li, M. Tian, Z. Zhen, Q. Dong, N. Kanwisher, and J. Liu. (2010). Heritability of the specific cognitive ability of face perception. Current Biology 20(2): 137-142.
https://www.sciencedirect.com/science/article/pii/S096098220902123X 

Thursday, June 27, 2019

The Original Industrial Revolution


Cro-Magnon woman (Wikicommons) – At northern latitudes, women had fewer opportunities for food gathering, so they were free to specialize in new and more cognitively demanding tasks, like garment making, needlework, weaving, leatherworking, pottery, and kiln operation.


I've published an article on the theory that cold Paleolithic winters selected for intelligence. This theory is often attributed to J. Philippe Rushton and Arthur Jensen but actually goes much further back. The article is open access (see link), and the abstract is provided below. Comments are welcome.


Rushton and Jensen argued that cognitive ability differs between human populations. But why are such differences expectable? Their answer: as modern humans spread out of Africa and into northern Eurasia, they entered colder and more seasonal climates that selected for the ability to plan ahead, in order to store food, make clothes, and build shelters for winter. This cold winter theory is supported by research on Paleolithic humans and recent hunter-gatherers. Tools become more diverse and complex as effective temperature decreases, apparently because food has to be obtained during limited periods and over large areas. There is also more storage of food and fuel and greater use of untended traps and snares. Finally, shelters have to be sturdier, and clothing more cold-resistant. The resulting cognitive demands are met primarily by women because the lack of opportunities for food gathering pushes them into more cognitively demanding tasks, like garment making, needlework, weaving, leatherworking, pottery, and kiln operation. The northern tier of Paleolithic Eurasia thus produced the "Original Industrial Revolution"—an explosion of creativity that preadapted its inhabitants for later developments, i.e., farming, more complex technology and social organization, and an increasingly future-oriented culture. Over time, these humans would spread south, replacing earlier populations that could less easily exploit the possibilities of the new cultural environment. As this environment developed further, it selected for further increases in cognitive ability. Indeed, mean intelligence seems to have risen during recorded history at temperate latitudes in Europe and East Asia. There is thus no unified theory for the evolution of human intelligence. A key stage was adaptation to cold winters during the Paleolithic, but much happened later.


Reference


Frost, P. (2019). The OriginalIndustrial Revolution. Did Cold Winters Select for Cognitive Ability? Psych 2019, 1(1), 166-181

https://doi.org/10.3390/psych1010012


Sunday, March 10, 2019

IQ of biracial children and adults


First snow in Minnesota (c. 1895), Robert Koehler. Biracial children have IQ scores halfway between those of white children and black children, even when they are conceived by white single mothers and adopted into middle-class white families in their first year of life.


You may have heard about the Minnesota Transracial Adoption Study. It was a longitudinal study of black, biracial, and white children adopted into white middle-class Minnesotan families, as well as the biological children of the same families (Levin, 1994; Lynn, 1994; Scarr and Weinberg, 1976; Weinberg, Scarr, and Waldman, 1992). IQ was measured when the adopted children were on average 7 years old and the biological children on average 10 years old. They were tested again ten years later. Between the two tests, all four groups declined in mean IQ. On both tests, however, the differences among the four groups remained unchanged, particularly the 15-point gap between black and white adoptees. 

The biracial children remained halfway between the black and white adoptees. Could this be due to the parental environment being likewise half and half? Well, no. All of them were raised by white parents, and they were adopted at an early age: 19 months on average for the white adoptees, 9 months for the biracial adoptees, and 32 months for the black adoptees. The last figure is emphasized by Scarr and Weinberg (1976) as a reason for the IQ gap between the black and white adoptees. 

Fine, but what about the IQ gap between the biracial and white adoptees? Almost all of the biracial children were adopted at a young age and born to white single mothers who had completed high school. From conception to adulthood they developed in a "white" environment. If anything, the white adoptees should have encountered more developmental problems because they were adopted at an older age.

Could color prejudice be a reason? Perhaps the biracial children were unconsciously treated worse than the white children. By the same reasoning, they may have been treated better than the black children. We can test the second half of this hypothesis. Twelve of the biracial children were wrongly thought by their adoptive parents to have two black parents. Nonetheless, they scored on average at the same level as the biracial children correctly classified by their adoptive parents (Scarr and Weinberg 1976).


The Eyferth study

Another study found no difference in IQ between white and biracial children. This was a study of children fathered by American soldiers in Germany and then raised by German mothers (Eyferth 1961). It found no significant difference in IQ between children with white fathers and children with black fathers. Both groups had a mean IQ of about 97.

These findings were criticized by Rushton and Jensen (2005) on three grounds:

1. The children were still young when tested. One third were between 5 and 10 years old and two thirds between 10 and 13. Since IQ is strongly influenced by family environment before puberty, a much larger sample would be needed to find a significant difference between the two groups.

2. Between 20 and 25% of the “black” fathers were actually North African.

3. At the time of the study, the US Army screened out low IQ applicants with its preinduction Army General Classification Test. The rejection rate was about 30% for African Americans and 3% for European Americans. African American soldiers are thus a biased sample of the African American population.

Another factor is that the capacity for intelligence seems to be more malleable in children than in adults. We see this with the Minnesota Transracial Adoption Study. In the enriched learning environment of middle-class Minnesota families, all of the children showed impressive IQ scores at 7 years of age. By 17 years of age, however, this benefit had largely washed out:

-------------------- Age 7 Age 17

Black children ----- 97 ----- 89

Biracial children - 109 ----- 99

White children --- 112 ---- 106

Does intelligence really decline with age because of wear and tear on the brain? Perhaps we’re programmed to be most intelligent in childhood. That’s when we have to familiarize ourselves with the world. The capacity for intelligence may then be gradually deactivated as we get older because it’s less necessary.

This deactivation may follow different trajectories in different human groups. In early Homo sapiens, it may have begun not long after puberty. As ancestral humans made the transition to farming, sedentary living, and increasingly complex societies, this learning capacity became more necessary in adulthood, with the result that natural selection favored those individuals who retained it at older ages. This gene-culture coevolution would have gone farther in some populations than in others.


The Fuerst et al study

A recent study led by John Fuerst has confirmed the intermediate IQ of biracial individuals, this time in adults. The research team used the General Social Survey, which includes not only ethnic, sociological, and demographic data but also a measure of intelligence (WordSum):


The relationship between biracial status, color, and crystallized intelligence was examined in a nationally representative sample of adult Black and White Americans. First, it was found that self-identifying biracial individuals, who were found to be intermediate in color and in self-reported ancestry, had intermediate levels of crystallized intelligence relative to self-identifying White (mostly European ancestry) and Black (mostly sub-Saharan African ancestry) Americans. The results were transformed to an IQ scale: White (M = 100.00, N = 7569), primarily White-biracial (M = 96.07, N = 43, primarily Black-biracial (M = 94.14 N = 50), and Black (M = 89.81, N = 1381).

The same study also found a significant negative correlation among African Americans between facial color and WordSum scores. The correlation was low (r = -0.102), but it would be difficult to get a higher correlation because of the measures used. Self-reported skin color correlates imperfectly with actual skin color, which in turn correlates imperfectly with European admixture. Wordsum likewise correlates imperfectly with IQ (r = 0.71). On a final note, the correlation between facial color and WordSum scores was not explained by region of residence, interviewer’s race, parental socioeconomic status, or individual educational attainment.


References

Eyferth, K. (1961). Leistungen verscheidener Gruppen von Besatzungskindern in Hamburg-Wechsler Intelligenztest für Kinder (HAWIK). Archiv für die gesamte Psychologie 113: 222-241.

Fuerst, J.G.R., R. Lynn, and E.O.W. Kirkegaard. (2019). The Effect of Biracial Status and Color on Crystallized Intelligence in the U.S.-Born African-European American Population. Psych 1(1): 44-54. https://dx.doi.org/10.3390/Psychology1010004

Levin, M. (1994). Comment on the Minnesota transracial adoption study. Intelligence 19: 13-20.

Lynn, R. (1994). Some reinterpretations of the Minnesota Transracial Adoption Study. Intelligence 19: 21-27.

Rushton, P. and A.R. Jensen. (2005). Thirty years of research on race differences in cognitive ability. Psychology, Public Policy, and Law 11: 235-294.

Scarr, S., and Weinberg, R.A. (1976). IQ test performance of Black children adopted by White families. American Psychologist 31: 726-739.

Weinberg, R.A., Scarr, S., and Waldman, I.D. (1992). The Minnesota Transracial Adoption Study: A follow-up of IQ test performance at adolescence. Intelligence 16: 117-135.

Tuesday, February 5, 2019

Did cold seasonal climates select for cognitive ability?


Paleolithic artefacts (Wikicommons). The northern tier of Eurasia saw an explosion of creativity that pre-adapted its inhabitants for later developments.


The new journal Psych will be publishing a special follow-up issue on J. Philippe Rushton and Arthur Jensen's 2005 article: "Thirty Years of Research on Race Differences in Cognitive Ability." The following is the abstract of my contribution. The article will appear later.


The first industrial revolution. Did cold seasonal climates select for cognitive ability?

Peter Frost

Abstract: In their joint article, Rushton and Jensen argued that cognitive ability differs between human populations. But why are such differences expectable? Their answer: as modern humans spread out of Africa and into the northern latitudes of Eurasia, they entered colder and more seasonal climates that selected for the ability to plan ahead, since they had to store food, make clothes, and build shelters for the winter. 

This explanation has a long history going back to Arthur Schopenhauer. More recently, it has been supported by findings from Paleolithic humans and contemporary hunter-gatherers. Tools become more diverse and complex as effective temperature decreases, apparently because food has to be obtained during limited periods of time and over large areas. There is also more storage of food and fuel and greater use of untended traps and snares. Finally, shelters have to be sturdier, and clothing more cold-resistant. The resulting cognitive demands fall on both men and women. Indeed, because women have few opportunities to get food through gathering, they specialize in more cognitively demanding tasks like garment making, needlework, weaving, leatherworking, pottery, and use of kilns. The northern tier of Paleolithic Eurasia thus produced the "first industrial revolution"—an explosion of creativity that pre-adapted its inhabitants for later developments, i.e., agriculture, more complex technology and social organization, and an increasingly future-oriented culture. Over time these humans would spread south, replacing earlier populations that could less easily exploit the possibilities of the new cultural environment. 

As this cultural environment developed further, it selected for further increases in cognitive ability. In fact, mean intelligence seems to have risen during historic times at temperate latitudes in Europe and East Asia. There is thus no unified theory for the evolution of human intelligence. A key stage was adaptation to cold seasonal climates during the Paleolithic, but much happened later.


References

Rushton, J.P. and A.R. Jensen. (2005). Thirty years of research on race differences in cognitive ability. Psychology, Public Policy, and Law 11(2): 235-294.


Saturday, January 3, 2015

Sometimes the consensus is phony


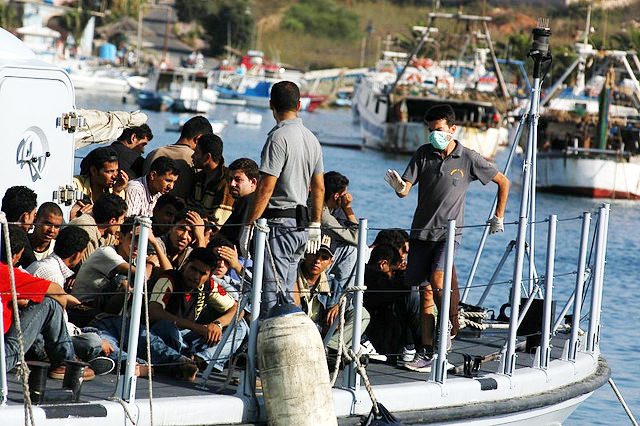
Migrants arriving on the island of Lampedusa (Wikicommons). The NATO-led invasion of Libya has opened a huge breach in Europe's defences.


A synthesis has been forming in the field of human biodiversity. It may be summarized as follows: 

1. Human evolution did not end in the Pleistocene or even slow down. In fact, it speeded up with the advent of agriculture 10,000 years ago, when the pace of genetic change rose over a hundred-fold. Humans were no longer adapting to relatively static natural environments but rather to faster-changing cultural environments of their own making. Our ancestors thus directed their own evolution. They created new ways of life, which in turn influenced who would survive and who wouldn't.

2. When life or death depends on your ability to follow a certain way of life, you are necessarily being selected for certain heritable characteristics. Some of these are dietary—an ability to digest milk or certain foods. Others, however, are mental and behavioral, things like aptitudes, personality type, and behavioral predispositions. This is because a way of life involves thinking and behaving in specific ways. Keep in mind, too, that most mental and behavioral traits have moderate to high heritability.

3. This gene-culture co-evolution began when humans had already spread over the whole world, from the equator to the arctic. So it followed trajectories that differed from one geographic population to another. Even when these populations had to adapt to similar ways of life, they may have done so differently, thus opening up (or closing off) different possibilities for further gene-culture co-evolution. Therefore, on theoretical grounds alone, human populations should differ in the genetic adaptations they have acquired. The differences should generally be small and statistical, being noticeable only when one compares large numbers of individuals. Nonetheless, even small differences, when added up over many individuals and many generations, can greatly influence the way a society grows and develops.

4. Humans have thus altered their environment via culture, and this man-made environment has altered humans via natural selection. This is probably the farthest we can go in formulating a unified theory of human biodiversity. For Gregory Clark, the key factor was the rise of settled, pacified societies, where people could get ahead through work and trade, rather than through violence and plunder. For Henry Harpending and Greg Cochrane, it was the advent of agriculture and, later, civilization. For J. Philippe Rushton and Ed Miller, it was the entry of humans into cold northern environments, which increased selection for more parental investment, slower life history, and higher cognitive performance. Each of these authors has identified part of the big picture, but the picture itself is too big to reduce to a single factor.

5. Antiracist scholars have argued against the significance of human biodiversity, but their arguments typically reflect a lack of evolutionary thinking. Yes, human populations are open to gene flow and are thus not sharply defined (if they were, they would be species). It doesn't follow, however, that the only legitimate objects of study are sharply defined ones. Few things in this world would pass that test.

Yes, genes vary much more within human populations than between them, but these two kinds of genetic variation are not comparable. A population boundary typically coincides with a geographic or ecological barrier, such as a change from one vegetation zone to another or, in humans, a change from one way of life to another. It thus separates not only different populations but also differing pressures of natural selection. This is why genetic variation within a population differs qualitatively from genetic variation between populations. The first kind cannot be ironed out by similar selection pressures and thus tends to involve genes of little or no selective value. The second kind occurs across population boundaries, which tend to separate different ecosystems, different vegetation zones, different ways of life ... and different selection pressures. So the genes matter a lot more.

This isn't just theory. We see the same genetic overlap between many sibling species that are nonetheless distinct anatomically and behaviorally. Because such species have arisen over a relatively short span of time, like human populations, they have been made different primarily by natural selection, so the genetic differences between them are more likely to have adaptive, functional consequences ... as opposed to "junk variability" that slowly accumulates over time.

Why is the above so controversial?

The above synthesis should not be controversial. Yet it is. In fact, it scarcely resembles acceptable thinking within academia and even less so within society at large. There are two main reasons.

The war on racism 

In the debate over nature versus nurture, the weight of opinion shifted toward the latter during the 20th century. This shift began during the mid-1910s and was initially a reaction against the extreme claims being made for genetic determinism. In reading the literature of the time, one is struck by the restraint of early proponents of environmental determinism, especially when they argue against race differences in mental makeup. An example appears in The Clash of Colour (1925), whose author condemned America's Jim Crow laws and the hypocrisy of proclaiming the rights of Europeans to self-determination while ignoring those of Africans and Asians. Nonetheless, like the young Franz Boas, he was reluctant to deny the existence of mental differences:

I would submit the principle that, although differences of racial mental qualities are relatively small, so small as to be indistinguishable with certainty in individuals, they are yet of great importance for the life of nations, because they exert throughout many generations a constant bias upon the development of their culture and their institutions. (Mathews, 1925, p. 151)

That was enlightened thinking in the 1920s. The early 1930s brought a radical turn with Hitler's arrival to power and a growing sense of urgency that led many Jewish and non-Jewish scholars to declare war on "racism." The word itself was initially a synonym for Nazism, and even today Nazi Germany still holds a central place in antiracist discourse.

Why didn't the war on racism end when the Second World War ended? For one thing, many people, feared a third global conflict in which anti-Semitism would play a dominant role. For another, antiracism took on a life of its own during the Cold War, when the two superpowers were vying for influence over the emerging countries of Asia and Africa.

Globalism

The end of the Cold War might have brought an end to the war on racism, or at least a winding down, had it not replaced socialism with an even more radical project: globalism. This is the hallmark of "late capitalism," a stage of historical development when the elites no longer feel restrained by national identity and are thus freer to enrich themselves at their host society's expense, mainly by outsourcing jobs to low-wage countries and by insourcing low-wage labor for jobs that cannot be relocated, such as those in construction and services. That's globalism in a nutshell.

This two-way movement redistributes wealth from owners of labor to owners of capital. Businesses get not only a cheaper workforce but also weaker labor and environmental standards. To stay competitive, workers in high-wage countries have to accept lower pay and a return to working conditions of another age. The top 10% are thus pulling farther and farther ahead of everyone else throughout the developed world. They're getting richer ... not by making a better product but by making the same product with cheaper and less troublesome inputs of labor. This is not a win-win situation, and the potential for revolutionary unrest is high.

To stave off unrest, economic systems require legitimacy, and legitimacy is made possible by ideology: a vision of a better future; how we can get there from here; and why we're not getting there despite the best efforts. Economic systems don't create ideology, but they do create conditions that favor some ideologies over others. With the collapse of the old left in the late 1980s, and the rise of market globalization, antiracism found a new purpose ... as a source of legitimacy for the globalist project.

I saw this up close in an antiracist organization during the mid to late 1980s. Truth be told, we mostly did things like marching in the May Day parade, agitating for a higher minimum wage, denouncing the U.S. intervention in Panama, organizing talks about Salvador Allende and what went wrong in Chile ... you get the drift. Antiracism was subservient to the political left. This was not a natural state of affairs, since the antiracist movement—like the Left in general—is a coalition of ethnic/religious factions that prefer to pursue their own narrow interests. This weakness was known to the political right, many of whom tried to exploit it by supporting Muslim fundamentalists in Afghanistan and elsewhere and black nationalists in Africa, Haiti, and the U.S. Yes, politics makes strange bedfellows.

With the onset of the 1990s, no one seemed to believe in socialism anymore and we wanted to tap into corporate sources of funding. So we reoriented. Leftist rhetoric was out and slick marketing in. Our educational materials looked glossier but now featured crude "Archie Bunker" caricatures of working people, and the language seemed increasingly anti-white. I remember feeling upset, even angry. So I left.

Looking back, I realize things had to happen that way. With the disintegration of the old socialist left, antiracists were freer to follow their natural inclinations, first by replacing class politics with identity politics, and second by making common cause with the political right, especially for the project of creating a globalized economy. Antiracism became a means to a new end.

This is the context that now frames the war on racism. For people in a position to influence public policy, antiracism is not only a moral imperative but also an economic one. It makes the difference between a sluggish return on investment of only 2 to 3% (which is typical in a mature economy) and a much higher one.

What to do?

Normally, I would advise caution. People need time to change their minds, especially on a topic as emotional as this one. When tempers flare, it's usually better to let the matter drop and return later. That's not cowardice; it's just a recognition of human limitations. Also, the other side may prove to be right. So, in a normal world, debate should run its course, and the policy implications discussed only when almost everyone has been convinced one way or the other.

Unfortunately, our world is far from normal. A lot of money is being spent to push a phony political consensus against any controls on immigration. This isn't being done in the dark by a few conspirators. It's being done in the full light of day by all kinds of people: agribusiness, Tyson Foods, Mark Zuckerberg, the U.S. Chamber of Commerce, and small-time operations ranging from landscapers to fast-food joints. They all want cheaper labor because they're competing against others who likewise want cheaper labor. It's that simple ... and stupid.

This phony consensus is also being pushed at a time when the demographic cauldron of the Third World is boiling over. This is particularly so in sub-Saharan Africa, where the decline in fertility has stalled and actually reversed in some countries. The resulting population overflow is now following the path of least resistance—northward, especially with the chaos due to the NATO-led invasion of Libya. In the current context, immigration controls should be strengthened, and yet there is lobbying to make them even weaker. The idiocy is beyond belief.

For these reasons, we cannot wait until even the most hardboiled skeptics are convinced. We must act now to bring anti-globalist parties to power: the UKIP in Britain, the Front national in France, the Partij voor de Vrijheid in the Netherlands, the Alternative für Deutschland in Germany, and the Sverigedemokraterna in Sweden. How, you may ask? It's not too complicated. Just go into the voting booth and vote. You don't even have to talk about your dirty deed afterwards. 

It looks like such parties will emerge in Canada and the United States only when people have seen what can be done in Europe. Until then, the tail must wag the dog. We in North America can nonetheless prepare the way by learning to speak up and stand up, and by recognizing that the "Right" is just as problematic as the "Left."
 

References


Clark, G. (2007). A Farewell to Alms. A Brief Economic History of the World, Princeton University Press, Princeton and Oxford. 

Clark, G. (2009a). The indicted and the wealthy: surnames, reproductive success, genetic selection and social class in pre-industrial England,
http://www.econ.ucdavis.edu/faculty/gclark/Farewell%20to%20Alms/Clark%20-Surnames.pdf 

Clark, G. (2009b). The domestication of Man: The social implications of Darwin, ArtefaCTos, 2(1), 64-80.
http://campus.usal.es/~revistas_trabajo/index.php/artefactos/article/viewFile/5427/5465 

Clark, G. (2010). Regression to mediocrity? Surnames and social mobility in England, 1200-2009
http://www.econ.ucdavis.edu/faculty/gclark/papers/Ruling%20Class%20-%20EJS%20version.pdf

Cochran, G. and H. Harpending. (2010). The 10,000 Year Explosion: How Civilization Accelerated Human Evolution, New York: Basic Books. 

Frost, P. (2011a). Human nature or human natures? Futures, 43, 740-748.
http://www.researchgate.net/publication/251725125_Human_nature_or_human_natures/file/504635223eaf8196f0.pdf  

Frost, P. (2011b). Rethinking intelligence and human geographic variation, Evo and Proud, February 11
http://evoandproud.blogspot.ca/2011/02/rethinking-intelligence-and-human.html 

Harpending, H., and G. Cochran. (2002). In our genes, Proceedings of the National Academy of Sciences U.S.A., 99, 10-12.
http://www.ncbi.nlm.nih.gov/pmc/articles/PMC117504/  

Hawks, J., E.T. Wang, G.M. Cochran, H.C. Harpending, and R.K. Moyzis. (2007). Recent acceleration of human adaptive evolution, Proceedings of the National Academy of Sciences U.S.A., 104, 20753-20758.
http://www.researchgate.net/publication/5761823_Recent_acceleration_of_human_adaptive_evolution/file/9c9605240c4bb57b55.pdf

Mathews, B. (1925). The Clash of Colour. A Study in the Problem of Race, London: Edinburgh House Press. 

Miller, E. (1994). Paternal provisioning versus mate seeking in human populations, Personality and Individual Differences, 17, 227-255.
http://www.prometheism.net/paternal/  

Rushton, J. P. (2000). Race, Evolution, and Behavior, 3rd ed., Charles Darwin Research Institute.
http://lazypawn.com/wordpress/wp-content/uploads/Race_Evolution_Behavior.pdf