Showing posts with label human evolution. Show all posts

Thursday, June 27, 2019

The Original Industrial Revolution


Cro-Magnon woman (Wikicommons) – At northern latitudes, women had fewer opportunities for food gathering, so they were free to specialize in new and more cognitively demanding tasks, like garment making, needlework, weaving, leatherworking, pottery, and kiln operation.


I've published an article on the theory that cold Paleolithic winters selected for intelligence. This theory is often attributed to J. Philippe Rushton and Arthur Jensen but actually goes much further back. The article is open access (see link), and the abstract is provided below. Comments are welcome.


Rushton and Jensen argued that cognitive ability differs between human populations. But why are such differences expectable? Their answer: as modern humans spread out of Africa and into northern Eurasia, they entered colder and more seasonal climates that selected for the ability to plan ahead, in order to store food, make clothes, and build shelters for winter. This cold winter theory is supported by research on Paleolithic humans and recent hunter-gatherers. Tools become more diverse and complex as effective temperature decreases, apparently because food has to be obtained during limited periods and over large areas. There is also more storage of food and fuel and greater use of untended traps and snares. Finally, shelters have to be sturdier, and clothing more cold-resistant. The resulting cognitive demands are met primarily by women because the lack of opportunities for food gathering pushes them into more cognitively demanding tasks, like garment making, needlework, weaving, leatherworking, pottery, and kiln operation. The northern tier of Paleolithic Eurasia thus produced the "Original Industrial Revolution"—an explosion of creativity that preadapted its inhabitants for later developments, i.e., farming, more complex technology and social organization, and an increasingly future-oriented culture. Over time, these humans would spread south, replacing earlier populations that could less easily exploit the possibilities of the new cultural environment. As this environment developed further, it selected for further increases in cognitive ability. Indeed, mean intelligence seems to have risen during recorded history at temperate latitudes in Europe and East Asia. There is thus no unified theory for the evolution of human intelligence. A key stage was adaptation to cold winters during the Paleolithic, but much happened later.


Reference


Frost, P. (2019). The OriginalIndustrial Revolution. Did Cold Winters Select for Cognitive Ability? Psych 2019, 1(1), 166-181

https://doi.org/10.3390/psych1010012


Saturday, August 2, 2014

Dear Fred


In a recent post, Fred Reed asks:


Why should I not indulge my hobby of torturing to death the severely genetically retarded? This would seem beneficial. We certainly don't want them to reproduce, they use resources better invested in healthy children, and it makes no evolutionary difference whether they die quietly or screaming.


The short answer is that any killing, for whatever reason, increases the likelihood of killing for other reasons. One exception is self-defence, but that's not done for pleasure. Another exception is capital punishment, but that, too, is not done for pleasure. More to the point, no single citizen can carry out an execution. It requires a lengthy judicial process. The same reasoning applies to the final exception of war. No single citizen can declare war.

It's not for nothing that killing is so taboo, especially recreational killing. Several things have contributed to the success of Western societies, but a leading one is the relatively peaceful nature of social relations. When people can go about their business without fearing for their lives, much becomes possible that otherwise would not be. This taboo is so crucial that we even extend it to nonhumans. Cats and dogs have no inherent right to life, yet it is a serious offence to torture them to death.
 

That's society. What about biology?

At this point, Fred may speak up: "But those are social reasons against killing of any sort. What are the biological reasons?"

The immediate biological reason is empathy. If I try to hurt someone, I feel the pain I inflict. Truth be told, the only life forms I enjoy killing are flies and mosquitoes. If a moth flies into our home, I'll go to some length to capture it and set it free outside, and I know others who do similar things. Just think of all the car drivers who come to a screeching halt to avoid running over some poor animal.

It's empathy that makes me and others act that way. And I cannot easily turn it off. It shuts down only when feelings of contempt enter my mind, as with those contemptible flies and mosquitoes.

Empathy is hardwired. It's 68% heritable in the case of affective empathy, i.e., the capacity to respond with the appropriate emotion to another person's mental state (Chakrabarti and Baron-Cohen, 2013). To date, studies have focused on disorders caused by too much empathy or too little. Psychopaths may have intact cognitive empathy, but impaired affective empathy. They keenly understand how others feel without actually experiencing those feelings. The reverse impairment may affect autists. As for depressives, they may suffer from being too sensitive to the distress of others and to guilt over not helping them enough. 

These disorders exist at the tail ends of a normal distribution. By focusing on these extremes, we forget the variability among healthy individuals. We all vary in our capacity for empathy, just as we do for almost any mental capacity.
 

How can evolution explain empathy?

Why do we feel empathy? How could natural selection favor such selflessness? This is of course the point that Fred is trying to make. Empathy keeps us from doing things that supposedly make evolutionary sense. Therefore, it could not have evolved. It must have been given to us by a Great Designer.

But why did this Great Designer give more of it to some people than to others? We're talking about a heritable trait. It's not as if everyone starts off the same way, with some later falling behind through their own wrongdoing.

And how has the Great Designer preserved this selfless behavior? Unless something is done, empathic people will eventually be overwhelmed by a tidal wave of cheaters, free riders, and people shouting "Gimme! Gimme! Gimme!" This is as much a mystery for creationists as it is for evolutionists. It's one thing to explain how altruism came to be. It's another to explain how it manages to survive in this cynical world.

These questions passed through my mind when I was going through my late mother's effects. I discovered she had for years been donating money for various projects in the Third World, at a time when she was a widow with no pension. Meanwhile, as a teenager, I had to take on all kinds of odd jobs to help us make ends meet. Looking over those donor receipts I shook my head and felt some resentment. How do good Christians like her manage to survive?

Yet she did, like others before her. For one thing, she was suspicious of strangers, and this suspicion extended to some ethnic groups more than to others. She was prejudiced and "postjudiced." If someone acted dishonestly with her once too often, she would have no more to do with him or her. Such people were "contemptible."

Today, that sort of behavior might seem un-Christian. But her Christianity was of an older, judgmental sort, being inspired more by the punitive Old Testament than by the forgiving New Testament. She would judge people, and her judgment could be harsh, very harsh.
 

Over space and time

Just as the capacity for empathy varies from one individual to another, it also varies statistically from one human population to another, being strongest in the "guilt cultures" of Northwest Europe. Guilt is the twin sister of empathy. Both flow from a simulation of how another person thinks or feels (an imaginary witness to a wrongdoing, a person in distress) and both ensure correct behavior by inducing the appropriate feelings (anguish, pity).

Why are guilt and empathy so strong in Northwest Europeans? Other societies ensure good behavior by relying on close kin to step in and enforce social rules. This policing mechanism has been less effective west of the Hajnal line (which runs roughly from Trieste to St. Petersburg) because kinship ties have been correspondingly weaker. There has thus been stronger selection for internal means of behavior control, like guilt and empathy.

This zone of relatively weak kinship is associated with unusual demographic tendencies, called the Western European Marriage Pattern:

- relatively late marriage for men and women

- many people who never marry

- neolocality (children leave the family household to form new households)

- high circulation of non-kin among different households (Hajnal, 1964; ICA, 2013)


The Western European Marriage Pattern was thought to have arisen after the Black Death of the 14th century. There is now good evidence for its existence before the Black Death and fragmentary evidence going back to 9th century France and earlier (Hallam, 1985; Seccombe, 1992, p. 94). Historian Alan Macfarlane likewise sees an English tendency toward weaker kinship ties before the 13th century and even during Anglo-Saxon times (Macfarlane, 2012; Macfarlane, 1992, pp. 173-174). I have argued that this tendency probably goes still farther back (Frost, 2013a; Frost, 2013b).
 

Whatever the ultimate cause, Northwest Europeans seem to have been pre-adapted for later shifts away from kinship and toward alternate means of organizing social relations (i.e., ideology, codified law, commerce). This tendency has taken various forms: the intense guilt-driven Christianity of the Anglo-Saxon penitential tradition and, later, Protestantism; the medieval alliance between Church and State to pacify social relations; and the post-medieval rise of the market economy. This cultural evolution has been described by the historical economist Gregory Clark for the English population between the 12th and 19th centuries. As England became a settled society, success went to those who could resolve disputes amiably and profit from thinking ahead—in short, those who had middle-class values of thrift, foresight, self-control, nonviolence, and sobriety. This English middle class, initially tiny, grew in numbers until its lineages accounted for most of its country’s gene pool (Clark, 2007; Clark, 2009a; Clark, 2009b).
 

But what does that have to do with evolution???
 
At this point, Fred may again speak up, with more than a touch of exasperation: "You're ducking my question! You're talking about culture, society, and religion! What does that have to do with evolution???"

Everything, Fred. Everything. Unlike other animals, humans have to adapt not only to their physical environment but also to their cultural environment. In short, we've become participants in our own evolution. We have domesticated ourselves.

Let me return to your initial question. What's to stop you from torturing to death the severely retarded? First, your sense of empathy should. If it doesn't, you're the one with a severe mental defect. I wouldn't want you as a fellow citizen, let alone as a neighbor. The law of the jungle may give you the right to torture defenceless people to death, but it also gives me the right to organize a lynch mob and hang you from the nearest tree.
 

References

Chakrabarti, B. and S. Baron-Cohen. (2013). Understanding the genetics of empathy and the autistic spectrum, in S. Baron-Cohen, H. Tager-Flusberg, M. Lombardo. (eds). Understanding Other Minds: Perspectives from Developmental Social Neuroscience, Oxford: Oxford University Press.

Clark, G. (2007). A Farewell to Alms. A Brief Economic History of the World, Princeton: Princeton University Press.

Clark, G. (2009a). The indicted and the wealthy: Surnames, reproductive success, genetic selection and social class in pre-industrial England.

Clark, G. (2009b). The domestication of man: The social implications of Darwin. ArtefaCTos, 2, 64-80.
http://campus.usal.es/~revistas_trabajo/index.php/artefactos/article/viewFile/5427/5465

Frost, P. (2013a). The origins of Northwest European guilt culture, Evo and Proud, December 7
http://evoandproud.blogspot.ca/2013/12/the-origins-of-northwest-european-guilt.html 

Frost, P. (2013b). Origins of Northwest European guilt culture, Part II, Evo and Proud, December 14
http://evoandproud.blogspot.ca/2013/12/origins-of-northwest-european-guilt.html

Hajnal, John (1965). European marriage pattern in historical perspective. In D.V. Glass and D.E.C. Eversley (eds). Population in History. Arnold, London.

Hallam, H.E. (1985). Age at first marriage and age at death in the Lincolnshire Fenland, 1252-1478, Population Studies, 39, 55-69. 

ICA (2013). Research Themes - Marriage Patterns, Institutions for Collective Action
http://www.collective-action.info/_THE_MarriagePatterns_EMP  

Macfarlane, A. (1992). On individualism, Proceedings of the British Academy, 82, 171-199.
http://www.alanmacfarlane.com/TEXTS/On_Individualism.pdf  

Macfarlane, A. (2012). The invention of the modern world. Chapter 8: Family, friendship and population, The Fortnightly Review, Spring-Summer serial
http://fortnightlyreview.co.uk/2012/07/invention-8/

Seccombe, W. (1992). A Millennium of Family Change. Feudalism to Capitalism in Northwestern Europe, London: Verso. 

Sunday, July 13, 2014

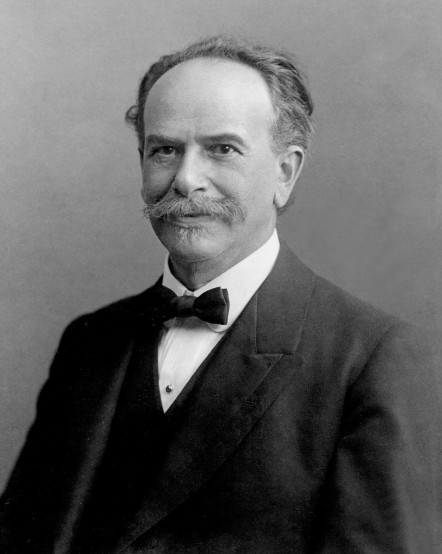
The Franz Boas you never knew


The anthropologist Franz Boas is remembered for moving the social sciences away from genetic determinism and toward environmental determinism. In reality, he felt that genes do contribute substantially to mental and behavioral differences ... and not just between individuals.


Most of us identify with certain great teachers of the past: Christ, Marx, Freud … Though long dead, they still influence us and we like to think that their teachings have come down to us intact. We know what they believed … or so we like to think. This raises a problem when we find discrepancies. Jesus was so humble that he resented being called good, since only God is truly good. But then ...

Often, however, the discrepancies remain unknown. They develop too gradually for the average person to notice and are most obvious to those who least want to point them out, i.e., the successors of the great teacher. Of course, the great teacher is no longer around to set things straight.

This has happened to many belief-systems. In my last post, I discussed how the real Sigmund Freud differed significantly from the one we know. The same is true for Franz Boas (1858-1942), whose school of anthropology is as much a product of his immediate disciples—Margaret Mead and Ruth Benedict—as of Boas himself.

Today, Boas is remembered as the man who moved the social sciences away from genetic determinism and toward environmental determinism. His Wikipedia entry states:

Boas was one of the most prominent opponents of the then popular ideologies of scientific racism, the idea that race is a biological concept and that human behavior is best understood through the typology of biological characteristics. [...] Boas also worked to demonstrate that differences in human behavior are not primarily determined by innate biological dispositions, but are largely the result of cultural differences acquired through social learning.

In reality, he felt that genes do contribute substantially to mental and behavioral differences ... and not just between individuals. This is apparent in a speech he gave in 1894 under the title "Human Faculty as Determined by Race."

It does not seem probable that the minds of races which show variations in their anatomical structure should act in exactly the same manner. Differences of structure must be accompanied by differences of function, physiological as well as psychological; and, as we found clear evidence of difference in structure between the races, so we must anticipate that differences in mental characteristics will be found.  [...] As all structural differences are quantitative, we must expect to find mental differences to be of the same description, and as we found the variations in structure to overlap, so that many forms are common to individuals of all races, so we may expect that many individuals will not differ in regard to their faculty, while a statistical inquiry embracing the whole races would reveal certain differences. Furthermore, as certain anatomical traits are found to be hereditary in certain families and hence in tribes and perhaps even in peoples, in the same manner mental traits characterize certain families and may prevail among tribes. It seems, however, an impossible undertaking to separate in a satisfactory manner the social and the hereditary features. Galton's attempt to establish the laws of hereditary genius points out a way of treatment for these questions which will prove useful in so far as it opens a method of determining the influence of heredity upon mental qualities (Boas, 1974, p. 239)

We have shown that the anatomical evidence is such, that we may expect to find the races not equally gifted. While we have no right to consider one more ape-like than the other, the differences are such that some have probably greater mental vigor than others. The variations are, however, such that we may expect many individuals of all races to be equally gifted, while the number of men and women of higher ability will differ. (Boas, 1974, p. 242) 

 When discussing brain size, Boaz merely pointed to the overlap among racial groups:

We find that 50 per cent of all whites have a capacity of the skull greater than 1550 cc., while 27 per cent of the negroes and 32 per cent of the Melanesians have capacities above this value. We might, therefore, anticipate a lack of men of high genius, but should not anticipate any great lack of faculty among the great mass of negroes living among whites and enjoying the advantages of the leadership of the best men of that race. (Boas, 1974, pp. 233-234)

He did add that "mental ability certainly does not depend upon the size of the brain alone." He then argued, quoting an authority, that the encephalon and the cortex develop to a greater degree in whites, especially after puberty:

When we compare the capacity for education between the lower and higher races, we find that the great point of divergence is at adolescence and the inference is fairly good that we shall not find in the brains of the lower races the post-pubertal growth in the cortex to which I have just alluded. (Boas, 1974, p. 234)

Boas would return to this topic, such as in this 1908 speech on "Race Problems in America":

I do not believe that the negro is, in his physical and mental make-up, the same as the European. The anatomical differences are so great that corresponding mental differences are plausible. There may exist differences in character and in the direction of specific aptitudes. There is, however, no proof whatever that these differences signify any appreciable degree of inferiority of the negro, notwithstanding the slightly inferior size, and perhaps lesser complexity of structure, of his brain; for these racial differences are much less than the range of variation found in either race considered by itself. (Boas, 1974, pp. 328-329)

All of these remarks must be judged in context. Boaz was trying to stake out a reasonable middle ground in opposition to the view that human races differ not only in degree but also in kind. There is also little doubt about his opposition to racial discrimination, which he felt was holding back many capable African Americans.

But he did not feel that equality of opportunity would lead to equality of results. This was the middle ground he defended, and it is far removed from today's middle ground. The two don't even overlap. What happened between then and now?

Something critical seems to have happened in the late 1930s. When Boas prepared the second edition of The Mind of Primitive Man (1938), he removed his earlier racialist statements. The reason was likely geopolitical. As a Jewish American seeing the rise of Nazi Germany, he may have felt that the fight against anti-Semitism would require a united front against all forms of “racism”—a word just starting to enter common use and initially a synonym for Nazism.

Boas died in 1942 and the leadership of his school of anthropology fell to Ruth Benedict and Margaret Mead. With the end of the war, both of them wished to pursue and even escalate the fight against racism. Escalation was favored by several aspects of the postwar era: lingering fears of a revival of anti-Semitism, competition between the two power blocs for the hearts and minds of the Third World, and an almost utopian desire to rebuild society—be it through socialism, social democracy, or new liberalism … In all this, we are no longer in the realm of science, let alone anthropology. 

Boas had sought to strike a new balance between nature and nurture in the study of Man. The war intervened, however, and Boasian anthropology was conscripted to fight not only the Axis but also racism in any form. Today, three-quarters of a century later, we’re still fighting that war.
 

References


Boas, F. (1974). A Franz Boas Reader. The Shaping of American Anthropology, 1883-1911, G.W. Stocking Jr. (ed.), Chicago: The University of Chicago Press. 

Wikipedia (2014). Franz Boas
http://en.wikipedia.org/wiki/Franz_Boas

Saturday, September 7, 2013

Why are we the naked ape?


Infant stump-tailed macaque (source). Other photos showing adults and infants (courtesy of Monte M. Taylor and Christopher H. Taylor).


Why do humans have so little body hair? This question is addressed by Sandel (2013) in his comparative review of hair density in 23 primates and 29 nonprimate mammals. There seems to have been a long-term trend towards hairlessness in our primate ancestors: 

[…] all primates, and chimpanzees in particular, are relatively hairless compared to other mammals. This suggests that there may have been selective pressures acting on the ancestor of humans and chimpanzees that led to an initial reduction in hair density. (Sandel, 2013)

Across species, hair density negatively correlates with body mass. This correlation may exist because bigger primates are of more recent origin. Or hairlessness may be a way to disperse the excess heat generated by a larger body, since the increase in surface area (and hence the ability to dissipate heat) does not keep pace with the increase in mass. Sandel rejects this ‘heat load’ hypothesis:

Wheeler (1984, 1985) hypothesized that the low hair density in humans was associated with increased sweating capabilities. If the low hair density among primates represents a thermoregulatory adaptation, there should be a negative correlation between eccrine sweat gland density and hair density. There are no comparative data on eccrine sweat gland density in primates, but the distribution of eccrine sweat glands (presence vs. absence in certain body regions) is not consistent with the thermoregulatory predictions (Montagna, 1972; Grant and Hoff, 1975). In sum, the negative relationship between hair density and body mass cannot currently be explained. (Sandel, 2013) 

He concludes that the evolutionary trend towards hairlessness cannot be due to anything specifically human, such as bipedality. Denudation of the skin must have begun even before the common ancestors of humans and chimpanzees went their separate ways:

If chimpanzees are indeed relatively hairless compared to other mammals, there may have been a selective pressure acting on the ancestor of humans and chimpanzees that led to an initial reduction in hair density. Current hypotheses for human hair evolution focus on uniquely human traits, such as bipedality or longdistance running. If a reduction in terminal hair density is shared with chimpanzees, we may need to develop hypotheses for human “hairlessness” based on traits that are shared among chimpanzees, bonobos, and humans. (Sandel, 2013). 

Social signaling?

One cause may have been a growing tendency among primates to replace fur coloration with skin coloration as a means to provide conspecifics with key information about oneself: age, sex, social rank, availability for mating, etc. (Higham, 2009). Increasingly complex social relations would have created more information to signal, thereby driving selection for denudation of the body surface. Since social status can change over a short span of time, skin might have edged out fur as a better way to convey this information to others.

In ancestral humans, the key signaler seems to have been the adult female, as Charles Darwin noted: 

As woman has a less hairy body than man, and as this character is common to all races, we may conclude that our female semi-human progenitors were probably first partially divested of hair; and that this occurred at an extremely remote period before the several races had diverged from a common stock. As our female progenitors gradually acquired this new character of nudity, they must have transmitted it in an almost equal degree to their young offspring of both sexes; so that its transmission, as in the case of many ornaments with mammals and birds, has, not been limited either by age or sex. […] 

The females of certain anthropoid apes, as stated in a former chapter, are somewhat less hairy on the under surface than are the males; and here we have what might have afforded a commencement for the process of denudation. (Darwin, 1871, pp. 377-378)

If we consider women’s skin, particularly its visual and tactile properties, it tends to be softer, smoother, paler, and more pliable. These are also the properties of infant skin. In this and other ways (e.g., face shape, pitch of voice), the adult female body tends to mimic the infant schema, perhaps as a way to trigger the same mental and behavioral responses. There may thus have been a three-stage evolutionary process where human skin lost its body hair through a selection pressure that first targeted infants and then women, with men becoming denuded as a side effect.

Infant skin color and social signaling

Primate infants use both skin and fur coloration to indicate their age class:

The coat color of the newborn infant of all species of Old World monkeys for which information is available is different from that of an adult of the same species. Often this difference is extremely striking, as in the dark-brown fur of the newborn langur. Skin color of the infant langur, baboon, and macaque is pink, in contrast to the almost black skin of the older infant or adult. The infant’s pink face, hands, and feet and its large pink ears are in sharp contrast to its dark brown fur. The natal coat color is present during the first two or three months of life, when the infant most needs protection and nourishment from its mother and older monkeys. It is almost certainly more than coincidence that the duration of coat color difference coincides with a period of dependency, when it is essential that the young be sheltered and protected by older animals (Jay, 1962)

According to a review of the primatological literature, the infant stage is most often identified by a specific fur color. Nonetheless, the infant does have differently colored skin in many species: “deep blue face colouration” (proboscis monkey), “white skin” (silvered leaf monkey), “pink/grey skin” (hanuman langur), “pink face” (spectacled leaf monkey), “pink skin” (capped langur), “pink face” (baboons), “pink flesh” (stump-tailed macaques), and “pale pink skin” (lion-tailed macaque) (Alley, 1980)

The skin seems to have reached its current denudation relatively late in hominid evolution, perhaps even after the fork that led on the one hand to Neanderthals and on the other to modern humans.  Neanderthals survived subzero climates without tailored clothing, and their sites yield only hide scrapers that could have served only to make blankets or ponchos. Microwear analysis shows that these scrapers were used for the initial phases of hide preparation, but not for the more advanced phases of clothing production (Hoffecker, 2002,p. 107). In contrast, modern human sites abound in eyed bone needles and bone awls (Hoffecker, 2002, pp. 107, 109, 135, 252). Further evidence for the relative lateness of tailored clothing is the recent origin of the human body louse, which lives in clothing and first appeared perhaps 83,000 to 170,000 years ago (Toups et al, 2011). Finally, Neanderthal infants seem to have clung to their mothers’ fur: “Chimpanzees have ridges on their finger bones that stem from the way that they clutch their mother’s fur as infants. Modern humans don’t have these ridges, but Neanderthals do” (Cochran and Harpending, 2009).

Denudation would have made the pale pink skin of infants visually more important. This pallor is striking in darker-skinned humans and seems to be appreciated by parents. A life story of a !Kung woman records why she would not kill her newborn child: “Uhn, Uhn … I don't want to kill her. This little girl is too beautiful. See how lovely and fair her skin is?” (Shostak, 2000, p. 70). In Kenya, newborn infants are often called mzungu ('European' in Swahili), and a new mother may tell her neighbors to come and see her mzungu (Walentowitz, 2008). Among the Tuareg, children are said to be born "white" because of the freshness and moisture of the womb (Walentowitz, 2008). The cause is often thought to be a previous spiritual life:

There is a rather widespread concept in Black Africa, according to which human beings, before "coming" into this world, dwell in heaven, where they are white. For, heaven itself is white and all the beings dwelling there are also white. Therefore the whiter a child is at birth, the more splendid it is. In other words, at that particular moment in a person's life, special importance is attached to the whiteness of his colour, which is endowed with exceptional qualities. (Zahan, 1974, p. 385)

Another Africanist makes the same point: "black is thus the color of maturity [...] White on the other hand is a sign of the before-life and the after-life: the African newborn is light-skinned and the color of mourning is white kaolin" (Maertens, 1978, p. 41).

Conclusion

Loss of body hair was a long-term evolutionary trend in ancestral hominids and even ancestral primates, being perhaps a response to a greater need for social signaling. In ancestral humans, the selection pressure seems to have gone through three stages, initially targeting infants and only later women and then men.

Among nonhuman primates, the relatively depigmented skin of infants has long exercised the signaling function of calming aggressive impulses in parents and stimulating protective, nurturing behavior. Women seem to have mimicked infant skin for the same purpose, perhaps because of the longer period of infant dependency and their correspondingly greater vulnerability during this period.

References

Alley, T.R. (1980). Infantile colouration as an elicitor of caretaking behaviour in Old World primates, Primates, 21, 416-429.
http://link.springer.com/article/10.1007/BF02390470#

Cochran, G. & H. Harpending (2009). Neanderthals, Steve Sailer’s iSteve Blog, January 10, 2009
http://isteve.blogspot.com/2009/01/neanderthals.html 

Darwin, C.R. (1871). The Descent of Man and Selection in relation to Sex, London: John Murray, vol. II, 1st edition.
http://darwin-online.org.uk/EditorialIntroductions/Freeman_TheDescentofMan.html 

Higham, J.P. (2009). Primate Coloration: An Introduction to the Special Issue, International Journal of Primatology, 30, 749–751.
http://link.springer.com/article/10.1007%2Fs10764-009-9381-y?LI=true# 

Hoffecker, J.F. (2002). Desolate Landscapes. Ice-Age Settlement in Eastern Europe, New Brunswick: Rutgers University Press.
http://books.google.fr/books?hl=fr&lr=&id=nXuqgInMOXIC&oi=fnd&pg=PR10&dq=Desolate+Landscapes.+Ice-Age+Settlement+in+Eastern+Europe&ots=UmwmLxMDDG&sig=bXfiayx_z0DSMQcwCauN5_8NHEw#v=onepage&q&f=false 

Jay, P.C. (1962). Aspects of maternal behavior among langurs, Annals of the New York Academy of Sciences, 102, 468-476.
http://onlinelibrary.wiley.com/doi/10.1111/j.1749-6632.1962.tb13653.x/abstract 

Maertens, J-T. (1978). Le dessein sur la peau. Essai d'anthropologie des inscriptions tégumentaires, Ritologiques I, Paris: Aubier Montaigne.

Sandel, A.A. (2013). Brief communication: Hair density and body mass in mammals and the evolution of human hairlessness, American Journal of Physical Anthropology, 152, 145–150.
http://onlinelibrary.wiley.com/doi/10.1002/ajpa.22333/abstract 

Shostak, M. (2000). Nisa: The Life and Words of a !Kung Woman, Harvard University Press.
http://books.google.fr/books?hl=fr&lr=&id=up4_q8ooKO0C&oi=fnd&pg=PP8&ots=IWCywpZQvq&sig=SaJsUdUZMeVTCGFFecXvD9mNVew#v=onepage&q&f=false 

Walentowitz, S. (2008). Des êtres à peaufiner. Variations de la coloration et de la pigmentation du nouveau-né, in J-P. Albert, B. Andrieu, P. Blanchard, G. Boëtsch, and D. Chevé (eds.) Coloris Corpus, (pp. 113-120), Paris: CNRS Éditions.

Zahan, D. (1974). White, Red and Black: Colour Symbolism in Black Africa, in A. Portmann and R. Ritsema (eds.) The Realms of Colour, Eranos 41 (1972), 365-395, Leiden: Eranos.

Saturday, August 20, 2011

Can evolutionary psychology evolve?

The Environment of Evolutionary Adaptedness, over a million years ago in the Pleistocene. A founding myth of evolutionary psychology.

In the future, how will we look at evolution and human behavior? Perhaps we’ll still be looking through the lens of evolutionary psychology, albeit a more “evolved” one than the current variety. Or perhaps there will be a new paradigm.

One thing is sure. Evolutionary psychology, as now defined, is untenable. It suffers from several flawed assumptions:

- Human nature is uniform, except for gender differences. It came into existence over a million years ago during the Pleistocene, in the Environment of Evolutionary Adaptedness (EEA). This was long before modern humans began to spread out of Africa some 40,000 years ago and eventually form the populations we know today.

- Given the complexity of human behavior, its genetic basis could not have changed to any appreciable extent since the Pleistocene.

- All present-day humans are therefore essentially the same. All differences in behavior, personality, and temperament must result from a single human nature responding to different environmental inputs.

These assumptions are false. Human genetic evolution has actually accelerated over the past 40,000 years, and even more so over the past 10,000. The latter period, in particular, was not one of people adapting to new physical environments defined by climate, landscape, and vegetation. People were adapting to new cultural environments defined by social structure, normative behavior, and technology.

Yes, human behavior is complex, and any genetic influences must be correspondingly complex. But these influences can be radically changed by a few point mutations. There’s no need to start from scratch, as John Tooby and Leda Cosmides imply. There may simply be changes to developmental timing, such as an infant’s mental plasticity being extended into older life stages. Or there may be changes to the degree of masculinization or feminization. The possibilities are endless. Again, there is no need to posit a huge number of genetic changes.

Yes, we are adapted to past environments—and not to the present one. And there is often a mismatch between something that made sense in the past and our present reality. But why assume a time gap of over one million years? Is it because the Pleistocene makes an ideal setting for just-so stories?

I suspect there is another, more cynical reason. By placing the evolutionary origins of human nature in the distant past, one avoids the messy reality of differences among current human populations—differences in outlook, personality, time orientation, and behavioral predisposition. The Pleistocene EEA may be a just-so story about the past, but it has also had a real impact on the present. It was part of the deal that made evolutionary psychology possible, in the wake of the firestorm that consumed sociobiology.

Will evolutionary psychology evolve?

A paradigm can evolve. Medicine was a pseudo-science that killed more patients than it cured as late as the 1920s. In the space of a few decades, the situation completely reversed. There have been similar turnarounds in other fields. Alchemy became chemistry, and astrology became astronomy.

Indeed, there have been calls for a rethinking of evolutionary psychology, even from Tooby and Cosmides. “Although the hominid line is thought to have originated on edges of the African savannahs, the EEA is not a particular place or time” (Tooby and Cosmides, 2005, p. 22). It is a composite of whichever selection pressures brought each adaptation into existence. There are thus potentially as many EEAs as there are adaptations, and some may be later than others.

This year, several evolutionary psychologists authored what may be called a manifesto for change:


We argue that the key tenets of the established EP paradigm require modification in the light of recent findings from a number of disciplines, including human genetics, evolutionary biology, cognitive neuroscience, developmental psychology, and paleoecology. For instance, many human genes have been subject to recent selective sweeps; humans play an active, constructive role in co-directing their own development and evolution; and experimental evidence often favours a general process, rather than a modular account, of cognition. (Bolhuis et al., 2011)

The text parallels my recent paper in Futures, sometimes strikingly so. It starts off by observing that in the early years of evolutionary psychology “our knowledge of the human genome was limited and gradualism dominated evolutionary thinking.” Today, we know differently:


Events in the Holocene (the last 10,000 years), particularly the adoption of agriculture, domestication of animals, and the increases in human densities that these practices afforded, were a major source of selection on our species, and possibly accelerated human evolution. Evidence from the human genome strongly suggests that recent human evolution has been affected by responses to features of the environment that were constructed by humans, from culturally facilitated changes in diet, to aspects of modern living that inadvertently promoted the spread of
diseases.
(Bolhuis et al., 2011)


This recent evolution has especially shaped the human brain: “Genes expressed in the human brain are well-represented in this recent selection.”

Even when assessed on its own terms, the Pleistocene EEA looks more and more like a myth, and should be treated as such:


[…] the abstract concept of stable selection pressures in the EEA is challenged by recent evidence from paleoecology and paleoanthropology. The Pleistocene was apparently far from stable, not only being variable, but progressively changing in the pattern of variation. The world experienced by members of the genus Homo in the early Pleistocene was very different from that experienced in the late Pleistocene, and even early anatomical modern Homo sapiens that lived around 150,000 years ago led very different lives from Upper Paleolithic people (40,000 years ago) (Bolhuis et al., 2011)


Is a paradigm shift in the offing? Probably. But what form will it take? Perhaps the second question is unimportant. Whether evolutionary psychology changes or disappears, we’ll be looking at evolution and human behavior in a very different light.

To be cont’d

References

Bolhuis, J.J., G.R. Brown, R.C. Richardson, and K.N. Laland. (2011). Darwin in mind: New opportunities for evolutionary psychology, PLoS Biol 9(7): e1001109. doi:10.1371/journal.pbio.1001109
http://www.plosbiology.org/article/info:doi/10.1371/journal.pbio.1001109

Frost, P. (2011). Human nature or human natures? Futures, 43, 740–748.
http://dx.doi.org/10.1016/j.futures.2011.05.017

Tooby, J. and L. Cosmides. (2005). Conceptual foundations of evolutionary psychology, in: D. M. Buss (Ed.) The Handbook of Evolutionary Psychology, Hoboken, NJ: Wiley, pp. 5-67.

Friday, January 14, 2011

On Neanderthals, Denisovans, and other archaics

Andaman Islanders. Related peoples once inhabited the coastal regions of southern, southeastern, and eastern Asia.

The past year brought two major advances: the long awaited sequencing of the Neanderthal genome and the genetic sequencing of an another archaic human, the Denisovans of East Asia, whose existence had previously been unsuspected.

The bottom line comes down to four points:

Before the East African ‘big bang’ gave rise to modern humans some 80,000 to 60,000 years ago, there had been at least four groups of archaic humans:

a) Skhul-Qafzeh hominins
- were almost modern anatomically
- were derived from a demic expansion that spread over most of Africa and the Middle East about 110,000 years ago
- evolved directly into modern humans through the rapid expansion of an East African subgroup

b) Neanderthals
- differed much more anatomically from modern humans
- were behaviorally similar to Skhul-Qafzeh hominins
- probably had body fur and other cold adaptations
- were derived from an earlier expansion out of Africa 250,000 - 400,000 years ago
- inhabited Europe, the Middle East (during glacial maxima), Central Asia, and Siberia as far east as Lake Baikal

c) Hobbits
- were small and possibly a form of Homo erectus
- inhabited at least a portion of southeast Asia
- may have been a regional variant of the Denisovans

d) Denisovans (Homo altaiensis?)
- were another archaic population distinct from modern humans
- inhabited Asia from Lake Baikal eastward (
see earlier post)

These archaic humans have left significant genetic admixture in all modern human populations. The admixture is about 1 to 4% in Eurasians (from Neanderthals), 8% in Melanesians (from Neanderthals and Denisovans), and 13% in sub-Saharan Africans (from Skhul-Qafzeh-like hominins).

This admixture might have accelerated human evolution by providing modern humans with useful alleles. To date, no such alleles have been found. The admixture seems to be confined to genes of low adaptive value.

Although Denisovans inhabited East Asia, they left no admixture in present-day East Asians. Yet their admixture is discernible in present-day Melanesians. It seems that the first modern humans to replace Denisovans were not ancestral East Asians but rather ancestral Melanesians. This is consistent with archeological and ethnographic evidence that the coastal regions of southern, southeastern, and eastern Asia were initially settled by people related to the indigenous populations of Melanesia, Papua-New Guinea, and Australia. After the last ice age, they were gradually replaced by populations originating in northern Eurasia (see earlier post). Today, they survive in relic groups like the Veddas of Sri Lanka, the Andaman Islanders, the Semang of the Malayan peninsula, and the Aeta of the Philippines.

References

Green, R.E., J. Krause, A.W. Briggs, T. Maricic, U. Stenzel, M. Kircher, et al. (2010). A draft sequence of the Neandertal genome, Science, 328, 710-722.
http://www.sciencemag.org/cgi/reprint/328/5979/710.pdf

Reich, D., R.E. Green, M. Kircher, J. Krause, N. Patterson, E.Y. Durand, et al. (2010). Genetic history of an archaic hominin group from Denisova Cave in Siberia." Nature, 468, 1053-1060.

Watson, E., P. Forster, M. Richards, and H-J. Bandelt. (1997). Mitochondrial footprints of human expansions in Africa, American Journal of Human Genetics, 61, 691-704.

Saturday, October 30, 2010

Did human evolution accelerate?

Modern humans changed little when they initially spread out of Africa and into the Middle East. Real change occurred farther north, when they entered seasonally varying environments that differed much more even in summer.

Three years ago, a research team led by John Hawks found that the rate of genetic change accelerated once ancestral humans had spread from Africa to the other continents. Over the past 40,000 years, natural selection seems to have altered at least 7% of our genome. And this process speeded up even more as agriculture replaced hunting and gathering over the past 10,000 years. The rate of genetic change then increased more than a hundred-fold (Hawks et al. 2007).

This finding, however, seems to be at odds with a recent Scientific American article by Jonathan Pritchard:

As early Homo sapiens spread out from Africa starting around 60,000 years ago, they encountered environmental challenges that they could not overcome with prehistoric technology.

Many scientists thus expected that surveys of our genomes would reveal considerable evidence of novel genetic mutations that have recently spread quickly through different populations by natural selection […]

But it turns out that although the genome contains some examples of very strong, rapid natural selection, most of the detectable natural selection appears to have occurred at a far slower pace than researchers had envisioned.
(Pritchard 2010)

Is there a fundamental disagreement here between Jonathan Pritchard and John Hawks? Perhaps not. Pritchard doesn’t actually deny that genetic change accelerated in ancestral humans. He simply states that its pace has been far slower than the one envisioned by “researchers.”

Curiously, he makes no reference to John Hawks. This is all the more curious because no one else matches the unnamed “many scientists” and “researchers.” Until three years ago, and even today, the conventional view has been that cultural evolution replaced genetic evolution in our species. Culture provided us with faster ways to adapt. Instead of changing our genes, we changed our environment by means of new technologies, modes of subsistence, forms of shelter, and so on.

That’s what I learned as an undergrad. If Pritchard wishes to argue against Hawks’ position, why not mention him by name? Why create a fictitious ‘conventional view’ that needs to be put in its place?

I see other weaknesses in this Scientific American article, particularly in the methodology behind its conclusion that human genetic evolution has been relatively slow. One is recognized by Pritchard himself. What matters is not the degree of change at a single gene, but rather the total change at all genes that influence a single trait:

A series of papers published in 2008, for example, identified more than 50 different genes that influence human height, and certainly many more remain to be found. For each of these, one allele increases average height by just three to five millimeters compared with the other allele.

When natural selection targets human height […] it may operate in large part by tweaking the allele frequencies of hundreds of different genes. If the “short” version of every height gene became just 10 percent more common, then most people in the population would quickly come to have more “short” alleles, and the population would be shorter overall.
(Pritchard 2010)

Another weakness is the impossibility of measuring the rate of genetic change directly:

It would be great if in our efforts to understand recent human evolution, we could obtain DNA samples from ancient remains and actually track the changes of favored alleles over time. (Pritchard 2010)

Because this approach is still in its infancy, Pritchard falls back on assumptions about when and where human populations have come into being. He assumes that Homo sapiens began to spread out of Africa some 60,000 years ago and then split into Europeans and East Asians some 20,000 to 30,000 years ago. These are the baselines he uses to calculate the rate of genetic change.

But these are high-end estimates. The ‘Out of Africa’ event is probably closer to 45,000 BP (1) and the best dating for the European/East Asian split is 20,000 BP (Laval et al. 2010) (2). Moreover, natural selection has not changed non-African humans at a constant rate since their ancestors left Africa. Those who remained within the tropical zone, such as Australian Aborigines, Papua-New Guineans, and Andaman Islanders, have changed surprisingly little. There has been much more evolution among those who spread out of the tropical zone and into temperate and arctic environments, beginning around 30,000 BP. Evolutionarily speaking, the key event was not when humans began to spread out of Africa. It was when they began to spread out of the Tropics (3).

So for many if not most traits, Pritchard is underestimating the rate of genetic change by a factor of two. Another source of error is his unspoken assumption that genetic change in Eurasia has never flowed back into Africa. By using Africa as a baseline for genetic change, he is excluding new Eurasian alleles that have displaced older ones even in Africa. Evidently, this error would lead to underestimation of the rate of genetic change both within and outside Africa.

Notes

1. Uranium dating suggests that modern humans entered the Middle East c. 46,500 BP (Schwarcz et al. 1979).

2. Maps of human prehistory typically show two lines of advance out of Africa: one turning left and into Europe and another turning right and into South Asia, Southeast Asia, and East Asia. The second line of advance did exist, but was not ancestral to present-day East Asians. It was instead ancestral to relic groups like the Andaman Islanders and the Semang, as well as Papua-New Guineans and Australian Aborigines.

East Asians, like the Inuit and Amerindians, have their origins in North Asia, as seen by their ‘Arctic’ physiognomy. These early North Asians in turn came from early Europeans, specifically the reindeer-hunting nomads who spread eastward through the steppe-tundra belt of northern Eurasia. In other words, Europeans and East Asians are not siblings who parted company in the Middle East some 45,000 years ago. The latter are instead ‘offspring’ of the former, the two groups having become reproductively isolated from each other at the height of the last ice age, c. 20,000 BP.

3. In sum, the ‘Out of Africa’ event did not occur when modern humans first ventured across the present-day Suez Canal. This is an arbitrary line based on current geopolitical realities. Ecologically speaking, the Middle East is part of Africa. Real adaptive change did not begin until modern humans had spread farther north and into environments with wide seasonal variations in temperature, vegetation, wildlife, and other resources.

References

Hawks, J., E.T. Wang, G.M. Cochran, H.C. Harpending, and R.K. Moyzis. (2007).
Recent acceleration of human adaptive evolution. Proceedings of the National Academy of Sciences (USA), 104, 20753-20758.

Laval, G., E. Patin, L.B. Barreiro, and L-Quintana-Murci. (2010). Formulating a historical and demographic model of recent human evolution based on resequencing data from noncoding regions, PloS ONE, 5(4), e10284

Pritchard, J.K. (2010). How we are evolving, Scientific American, October, pp. 41-47.

Schwarcz, H.P., B. Blackwell, P. Goldberg, and A.E. Marks. (1979). Uranium series dating of travertine from archaeological sites, Nahal Zin, Israel, Nature, 277, 558-560.

Thursday, April 22, 2010

The puzzle of European hair and eye color


I’ve been fascinated by a puzzle of modern human evolution: the diverse palette of hair and eye colors that has developed in some populations (Frost, 2006; Frost 2008). Hair may be black, brown, flaxen, golden, or red, and eyes may be brown, blue, gray, hazel, or green. Both polymorphisms are largely confined to Europeans, especially those from the north and east.

This is an evolutionary puzzle for several reasons:

1. Hair color and eye color diversified through two separate processes that involved several gene loci (principally at MC1R for hair color and at OCA2-HERC2 for eye color).

2. Both processes occurred within the same geographic area.

3. Both processes occurred within a relatively narrow time frame, i.e., after the arrival of modern humans in Europe c. 35,000 years ago. Current estimates place this evolutionary change quite late in time, perhaps during the last ice age (25,000 - 10,000 BP).

For some anthropologists, this palette of hair and eye colors is a side effect of the lighter skin of Europeans. This lighter skin is, in turn, due to relaxation of selection for dark skin at non-tropical latitudes and a resulting accumulation of ‘loss of function’ alleles that affect not only skin color but also hair and eye color.

Yet relaxation of selection could not have produced so many new alleles over so little time. If selection is relaxed at loci for hair and eye color, close to a million years must elapse to produce the hair- and eye-color variability that Europeans now display, including ~ 80,000 years for the current prevalence of red hair alone (Harding et al., 2000; Templeton, 2002). This is much longer than the c. 35,000 years that modern humans have been in Europe. Moreover, the presumed initial cause—the whitening of European skin—seems to have occurred long after the arrival date of 35,000 BP (Norton & Hammer, 2007). As a Science journalist commented: “the implication is that our European ancestors were brown-skinned for tens of thousands of years” (Gibbons, 2007).

The puzzle is not resolved if Europeans turned white because of positive selection for lighter skin, as opposed to relaxation of selection for darker skin. Such a scenario would not have caused hair and eye color to diversify. In fact, most of the new alleles have little or no relationship with skin color. Only red hair and blue eyes are visibly associated with lighter skin.

There must have been positive selection for diversity of hair and eye color in and of itself. And this selection must have been very strong, given the relatively narrow time frame.

I have suggested that the likeliest explanation is sexual selection (Frost, 2006; Frost, 2008). This kind of explanation is consistent with several general facts:

1. Sexual selection typically creates brightly colored traits.

2. Such traits tend to be on or close to the face, because this part of the body attracts the most visual attention.

3. Intense sexual selection can produce color polymorphisms.

But why would sexual selection have been stronger among northern and eastern Europeans than among other human populations? To answer this question, we must understand why sexual selection should have differed in intensity among ancestral modern humans. In general, the differences were latitudinal, i.e., sexual selection differed primarily along a north-south axis.

Latitudinal differences in the ratio of men to women on the mate market

In the tropical zone, a woman could gather or grow enough food for herself and her children with little assistance. Because the cost of providing for a second wife was very low (often negative, i.e., a net gain), a man’s optimal reproductive strategy was to have as many wives as possible. There were thus too many men competing for too few women.

The farther away ancestral humans were from the tropics, the more women needed food (meat) provided by men. This was especially so in winter, when opportunities for food gathering were scarce. The cost of providing for a second wife was thus high, making polygyny impossible for all but the ablest hunters.

Alongside this trend of increasing female dependence on male providers was another north-south trend: male mortality increased farther away from the tropics because of longer hunting distances and the resulting increased risk of death due to accidents, exposure, starvation, etc.

Continental Arctic: optimal conditions for sexual selection of women

These two trends culminated in the continental Arctic. Here, women had few opportunities for food gathering at any time of year. They and their children depended almost wholly on meat that men provided through hunting. Here too, hunting distance was at a maximum. Men hunted wandering herds of herbivores, mainly reindeer, over very long distances. The high rate of male mortality, combined with the low rate of polygyny, limited the number of males available for mating. Result: a corresponding surplus of unmated females and intense sexual selection of women.

Today, this kind of environment is confined to the northern fringes of Eurasia and North America, but during the last ice age (25,000 – 10,000 BP) it lay further south and covered more territory. This was especially so in Europe, where the Scandinavian icecap had pushed the steppe-tundra zone down to the plains stretching from southwestern France through northern Germany and into eastern Europe. These temperate latitudes permitted a high level of bioproductivity and a comparatively large human population—the ancestors of today’s Europeans.

Sexual selection and color traits

When sexual selection is weak, the adaptive equilibrium is dominated by selection for a dull, cryptic appearance that reduces detection by predators. As sexual selection grows stronger, the equilibrium shifts toward a more noticeable appearance that retains the attention of potential mates, typically by means of vivid and/or novel colors.

One outcome may be a polymorphism of brightly colored phenotypes, due to the pressure of selection shifting to scarcer and more novel hues whenever a color variant becomes too common. This frequency dependence has been shown in humans. Thelen (1983) presented male participants with slides showing attractive brunettes and blondes and asked them to choose, for each series, the woman they would most like to marry. One series had equal numbers of brunettes and blondes, a second 1 brunette for every 5 blondes, and a third 1 brunette for every 11 blondes. Result: the rarer the brunettes were in a series, the likelier any one brunette would be chosen.

Among ancestral Europeans, this selection pressure may have caused a proliferation of new hair and eye colors to the detriment of our species norm of black hair and brown eyes. The selection was partly for novel colors. A rare color engages visual attention for a longer time than does a more common color (Brockmole & Boot, 2009). It may be that color rarity stimulates a mental algorithm that scans the visual environment for new or unusual objects.

In addition to color novelty, there also seems to have been selection for color brightness. Hair is carrot-red but not burgundy red. Eyes are light blue but not navy blue. Maan and Cummings (2009) argue that brighter colors have a stronger impact because they deliver a stronger signal that is more readily learned and retained in memory.

In a mate market already saturated with high-quality females, these eye-catching characteristics—color novelty and color brightness—may have made the difference between success and failure in finding a mate.

Other evidence for unusually strong sexual selection of European women

Hair and eye color polymorphism coincide geographically with other unusual physical traits. There is, for instance, the extreme whitening of the skin, which we do not see in other human populations at similar latitudes and which may have been driven by male targeting of lighter skin as a female-specific characteristic.

There also seems to have been selection to accentuate female-specific traits. Women of European descent have wider hips, narrower waists, and thicker deposition of subcutaneous fat than do women of other geographic origins (Hrdlička, 1898; Meredith & Spurgeon, 1980; Nelson & Nelson, 1986). Even before birth, Euro-American fetuses show significantly more sexual dimorphism than do African-American fetuses (Choi & Trotter, 1970).

In the same vein, Liberton (2009) has found that face shape differentiated between Europeans and sub-Saharan Africans in part through a selective force that has acted primarily on women, and not on both sexes. This too would be consistent with the selection pressure that seems to have diversified European hair and eye color.

References

Brockmole, J.R. & W.R. Boot. (2009). Should I stay or should I go? Attentional disengagement from visually unique and unexpected items at fixation, Journal of Experimental Psychology, 35, 808-815.

Choi, S.C., & Trotter, M. A. (1970). Statistical study of the multivariate structure and race‑sex differences of American White and Negro fetal skeletons. American Journal of Physical Anthropology, 33, 307‑312.

Frost, P. (2008). Sexual selection and human geographic variation, Proceedings of the 2nd Annual Meeting of the NorthEastern Evolutionary Psychology Society, The Journal of Social, Evolutionary & Cultural Psychology, 2 (supp.), 49-65,
www.jsecjournal.com/NEEPSfrost.pdf

Frost, P. (2006). European hair and eye color - A case of frequency-dependent sexual selection? Evolution and Human Behavior, 27, 85-103
http://www.sciencedirect.com/science/journal/10905138

Gibbons, A. (2007). American Association Of Physical Anthropologists Meeting: European Skin Turned Pale Only Recently, Gene Suggests. Science 20 April 2007: 316. no. 5823, p. 364 DOI: 10.1126/science.316.5823.364a
http://www.sciencemag.org/cgi/content/summary/316/5823/364a

Harding, R.M., Healy, E., Ray, A.J., Ellis, N.S., Flanagan, N., Todd, C., Dixon, C., Sajantila, A., Jackson, I.J., Birch‑Machin, M.A., & Rees, J.L. (2000). Evidence for variable selective pressures at MC1R. American Journal of Human Genetics, 66, 1351‑1361.

Hrdlička, A. (1898). Physical differences between White and Colored children. American Anthropologist, 11, 347‑350.

Liberton, D.K., K.A. Matthes, R. Pereira, T. Frudakis, D.A. Puts, & M.D. Shriver. (2009).
Patterns of correlation between genetic ancestry and facial features suggest selection on females is driving differentiation. Poster #326, The American Society of Human Genetics, 59th annual meeting, October 20-24, 2009. Honolulu, Hawaii.

Maan, M.E. & M.E. Cummings. (2009). Sexual dimorphism and directional sexual selection on aposematic signals in a poison frog, Proceedings of the National Academy of Sciences (USA), 106, 19072-10977.

Meredith, H.V., & Spurgeon, J.H. (1980). Somatic comparisons at age 9 years for South Carolina White Girls and girls of other ethnic groups. Human Biology, 52, 401‑411.

Nelson, J.K., & Nelson, K.R. (1986). Skinfold profiles of Black and White boys and girls ages 11‑13. Human Biology, 58, 379‑390.

Norton, H.L. & Hammer, M.F. (2007). Sequence variation in the pigmentation candidate gene SLC24A5 and evidence for independent evolution of light skin in European and East Asian populations. Program of the 77th Annual Meeting of the American Association of Physical Anthropologists, p. 179.

Templeton, A.R. (2002). Out of Africa again and again. Nature, 416, 45-51.

Thelen, T.H. (1983). Minority type human mate preference. Social Biology, 30, 162-180.